Abstract
There are only two classes of small-molecule drugs for infectious disease: pathogen-directed antimicrobials and host-directed immunomodulators. The former includes antibiotics and antivirals while the latter comprises corticosteroids such as dexamethasone. Here I inaugurate a third class, immunomodulatory antimicrobials (IAs), which considers small-molecule drugs harbouring both pathogen-directed and host-directed pharmacology. I review seven types of IAs, and argue that their high repositionability and network pharmacological ability to counter multiple pathogen types render them more applicable to pandemic-preparedness research than antivirals.
Keywords: Immunomodulatory antimicrobial, Pan-pathogen pharmacology, Pandemic preparedness
1. Introduction
It is said, that on his deathbed, Louis Pasteur retracted his germ theory of disease. Conceding, ‘Le microbe n’est rien, le terrain est tout’ (The microbe is nothing, the terrain is everything), Pasteur had spent decades propagating the idea that pathogens are the cause of infectious disease [1 (opens in a new tab)]. In contrast, the terrain theory (or host theory), championed by Pasteur’s contemporaries Claude Bernard and Antione Béchamp, contended that an unhealthy bodily environment causes disease [2 (opens in a new tab)].
In the 20th century, Paul Ehrlich’s ‘magic bullet’ concept complemented Pasteur’s work by defining a treatment development paradigm for infectious diseases based upon using small-molecule drugs to kill pathogens [3 (opens in a new tab)]. From the discovery of penicillin in the 1920s to the development of antivirals in recent decades, the magic bullet paradigm is a century-spanning success in combatting the plethora of pathogens that cause disease [4 (opens in a new tab)5 (opens in a new tab)]. Contemporary antimicrobial nomenclature still reflects this pathogen-centred approach: the term ‘antibiotic’ derives from the Greek αντι anti, ‘against’ and βíoc bios, ‘life’ - literally ‘opposing life’ [6 (opens in a new tab)].
The most well-known limitation of the magic bullet approach to antimicrobial development is the concomitant rise of antimicrobial resistance (AMR) over the last century, which has occurred in all pathogen classes [7 (opens in a new tab)]. The second limitation has only come to light recently, when the 2020 pandemic saw the emergence of a novel infectious disease unabated by existing pharmaceuticals [8 (opens in a new tab)]. While it was hoped that antiviral drugs such as remdesivir would be effective against the novel disease, instead the small-molecule corticosteroid dexamethasone arose as a successful host-directed approach to treat severe COVID-19: the first ‘magic shield’ [9 (opens in a new tab)].
The need to develop immunomodulators to prepare against novel infectious diseases is not a new argument: in 1987 Stanley Wiener envisioned the use of ‘broad-spectrum… agents that enhance the immune system [to] provide a non-specific, but effective, medical defense in the future’ [10 (opens in a new tab)]; in 2007, the Strategic Plan for Biodefense Research by the U.S. Department of Health and Human Services described the need for general emergency pills for global health crises [11 (opens in a new tab)]. By targeting the host immune system instead of a specific pathogen, therapeutics could indeed become ‘non-specific’ insofar as being deployable against a range of pathogens. The broader the pathogen range of a therapeutic, the more suitable for ‘Pathogen X’, a hypothetical, unknown pathogen that could cause a future epidemic. Likewise, ‘Drug X’, a hypothetical therapeutic that is repositionable against the widest range of pathogen types, must harbour an equally broad pharmacological profile in anticipation of novel diseases.
I have discovered two classes of host-modulating drugs that display efficacy against multiple pathogen classes, a pharmacological property hereby termed ‘pan-pathogen pharmacology’ (PPP). The first is small-molecule immunomodulators such as dexamethasone, whose success in treating both bacterial infections as well as COVID-19 underscores the notion that immunomodulators can treat infectious disease across pathogen classes [12 (opens in a new tab)]. The second is pathogen-inhibiting antimicrobials which also exhibit immunomodulatory activity, henceforth termed ‘immunomodulatory antimicrobials’ (IAs) [13 (opens in a new tab)]. As with typical antimicrobials and immunomodulators, IAs shift the damage-response curve towards reducing damage to the host [14 (opens in a new tab)]. However, they exhibit both pathogen-directed and host-modulating capabilities: a polypharmacological property which bestows their propensity to treat disease across pathogen classes [15 (opens in a new tab)].
This review contends that the magic shield must supersede the magic bullet as the goal of antimicrobial development. While recognition of the magic shield paradigm confutes Ehrlich’s magic bullet, it addresses AMR and COVID-19, reinstitutes Bernard and Béchamp’s terrain theory, and unlocks the possibility of developing a single drug for all infectious disease, both extant and emergent [16 (opens in a new tab)].
2. IAs
Although both IAs and magic shields exhibit PPP, the PPP for IAs is more assiduously characterised. Magic shields like dexamethasone, while useful for treating bacterial meningitis and COVID-19, have long been known to exacerbate symptoms when used to treat other infection types [17 (opens in a new tab)]. Instead, the unique bullet/shield network pharmacology of IAs appears to underscore their applicability for a broader range of communicable diseases. The pharmacology of seven classes of IAs is henceforth discussed: tetracyclines, quinolines, sesquiterpene lactones, fluoroquinolones, benzimidazoles, macrolides, and salicylanilides (Fig. 1 (opens in a new tab) ).
Click on image to zoom (opens in a new tab)
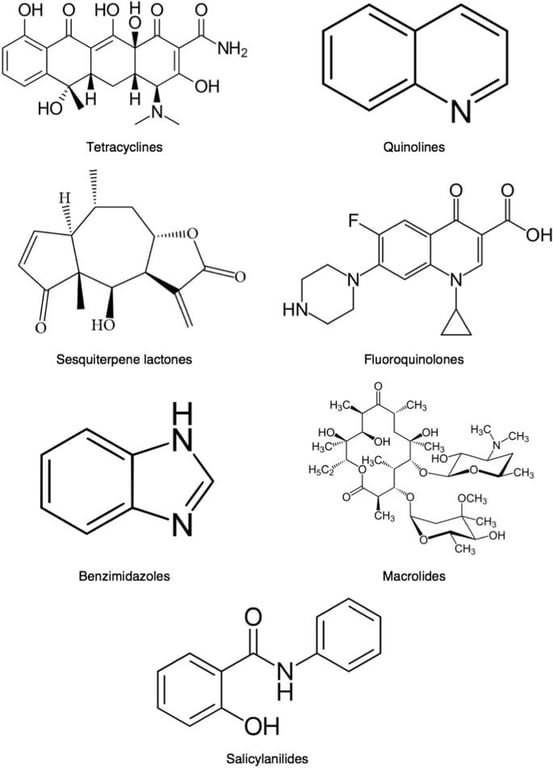
Seven classes of IAs. IAs comprise a heterogeneous subset of compounds which display both pathogen-killing (magic bullet) and host-directed (magic shield) properties. This hallmark is achieved by polypharmacological perturbation of signalling networks within the host-pathogen interactome (network pharmacology).
2.1. Tetracyclines
The first IA class comprises the oldest antibiotics. Discovered in the 1940s, tetracyclines are the archetypal antibiotics that have been repositioned against a variety of disease types from malaria to cancer, all while their magic shield pharmacological profiles are ascertained [[18] (opens in a new tab), [19] (opens in a new tab), [20] (opens in a new tab), [21] (opens in a new tab), [22] (opens in a new tab), [23] (opens in a new tab), [24] (opens in a new tab)].
The magic bullet properties of tetracyclines are well characterised [25 (opens in a new tab)]. They inhibit protein synthesis of bacteria by binding reversibly to the bacterial 30 S ribosomal subunit and preventing the aminoacyl tRNA from binding to the A site of the ribosome [26 (opens in a new tab)]. They also partially bind the bacterial 50 S ribosomal subunit and may alter the cytoplasmic membrane to cause intracellular components to leak from bacterial cells [27 (opens in a new tab)28 (opens in a new tab)]. With regard to malarial infection, tetracyclines block expression of the apicoplast genome, driving distribution of non-functional apicoplasts into daughter merozoites and leading to a potent antimalarial effect [29 (opens in a new tab)30 (opens in a new tab)].
The development of immunomodulatory tetracyclines, such as doxycycline and minocycline, is a breakthrough in antibiotic therapy and recent investigations have shed light on their mechanisms of action [31 (opens in a new tab)32 (opens in a new tab)]. Both potentiate the innate immune response and incite resolution of inflammation [33 (opens in a new tab)34 (opens in a new tab)]. Immunomodulatory tetracyclines were recently shown to potentiate macrophage cytokine release in vitro, and while improving mucosal recovery in colitic mice, minocycline enhanced pro-inflammatory cytokine release, including IL-1β, IL-6, and IL-4, in contrast to macrolides which dampen the cytokine storm. However, there is also evidence of the ability of minocycline to reduce pro-inflammatory cytokine release in non-communicable diseases, warranting further investigations [35 (opens in a new tab)].
Overall, the magic shield properties of tetracyclines, manifesting as a plethora of mechanisms modulating host immune pathways, reposition this drug class to an equally broad range of disease states [[36] (opens in a new tab), [37] (opens in a new tab), [38] (opens in a new tab), [39] (opens in a new tab), [40] (opens in a new tab), [41] (opens in a new tab)]. Indeed, the study of tetracyclines as antivirals is over 50 years old, with the first available report on their antiviral activity being published by Negrette et al. in the 1960s [42 (opens in a new tab)]. More recently, a range of tetracycline antibiotics were inducted into clinical trials for COVID-19 due to their ability to chelate and inhibit host matrix metalloproteinases (MMPs) which are co-opted by RNA viruses [[43] (opens in a new tab), [44] (opens in a new tab), [45] (opens in a new tab), [46] (opens in a new tab), [47] (opens in a new tab), [48] (opens in a new tab), [49] (opens in a new tab)]. Lastly, a combination of tetracycline and a macrolide (another IA class) has been suggested as a possible treatment regimen for COVID-19, intimating the potential benefits of combinatorial IA treatment [50 (opens in a new tab)].
2.2. Quinolines
Comparable with the clinical history of tetracyclines for bacterial diseases is the clinical history of quinolines for malaria. A heterocyclic aromatic organic compound, quinoline is characterised by a double-ring structure containing a benzene ring fused to pyridine at two adjacent carbon atoms [51 (opens in a new tab)]. While quinoline itself has few applications, its derivatives exhibit broad antimalarial and anticancer activity [52 (opens in a new tab)53 (opens in a new tab)].
Quinolines are magic bullets against bacteria, malaria, and fungi. Nitroxoline (8-hydroxy-5-nitroquinoline) is an 8-hydroxyquinoline derivative that has been prescribed as an antibiotic for decades in Europe to treat urinary tract infections, its antibiotic activity being attributed to its ability to chelate metal ions (akin to tetracyclines) and to dispel biofilms [54 (opens in a new tab)]. Chloroquine is a protonated, weakly basic 4-aminoquinoline that accumulates in the food vacuole of parasites and interferes with degradation of host red blood cell (RBC) haemoglobin, preventing malarial parasite growth [[55] (opens in a new tab), [56] (opens in a new tab), [57] (opens in a new tab)]. Unmodified quinoline exhibits relatively high activity against some fungal strains at non-toxic concentrations and the fungistatic activity of 8-hydroxyquinoline and its metal complexes has been known since the early 1920s, with these compounds now broadly used in healthcare [58 (opens in a new tab)].
2020 saw many reviews highlighting the immunomodulatory activities of chloroquine and hydroxychloroquine [59 (opens in a new tab)60 (opens in a new tab)]. At concentrations less than 20 μM, both inhibit activation of nucleic acid sensors, Toll-like receptors (TLRs) in endosomes, and cyclic GMP-AMP synthase (cGAS) in the cytoplasm [61 (opens in a new tab)]. This leads to inhibition of pattern recognition receptor (PRR)-induced activation of downstream pro-inflammatory cytokine and type I interferon (IFN) gene expression [62 (opens in a new tab)]. At concentrations higher than 100 μM, chloroquine and hydroxychloroquine increase lysosomal pH, leading to disruption of presentation of extracellular antigens processed through the endolysosomal pathway and intracellular antigens processed through the autophagosome-lysosome fusion pathway by antigen presenting cells [63 (opens in a new tab)64 (opens in a new tab)]; this property, revisited in Section 3 (opens in a new tab), is a prospective hallmark of IAs. The extensive magic shield pharmacology of quinolines has likely contributed to their use as antiproliferative agents [[65] (opens in a new tab), [66] (opens in a new tab), [67] (opens in a new tab), [68] (opens in a new tab), [69] (opens in a new tab), [70] (opens in a new tab), [71] (opens in a new tab), [72] (opens in a new tab), [73] (opens in a new tab), [74] (opens in a new tab)]. Overall, recognition that quinolines are IAs affirms the untapped repositioning potential of these antiparasitic agents for cancer, viral pandemics, and bacterial and fungal infection [[75] (opens in a new tab), [76] (opens in a new tab), [77] (opens in a new tab), [78] (opens in a new tab), [79] (opens in a new tab), [80] (opens in a new tab), [81] (opens in a new tab)].
2.3. Sesquiterpene lactones
As chloroquine was first extracted from the bark of Cinchona officinalis trees, so sesquiterpene lactones have been extracted from Artemisia annua wormwood plants. Sesquiterpenes are a class of terpenes that consist of three isoprene units; sesquiterpene lactones are a class of sesquiterpenes that contain a lactone ring [82 (opens in a new tab)]. Artemisinin, a new, highly effective antimalarial compound, is a sesquiterpene lactone found in Artemisia annua [83 (opens in a new tab)]. It was discovered in 1972 by Tu Youyou, who shared the 2015 Nobel Prize in Physiology or Medicine for its discovery [84 (opens in a new tab)].
Artemisinin-based combination therapies (ACTs) are considered standard treatment worldwide for P. falciparum malaria as well as malaria due to other species of Plasmodium [85 (opens in a new tab)]. Artemisinin’s mechanism of action includes induction of oxidative stress in infected RBCs [86 (opens in a new tab)]. However, evidence of artemisinin resistance was discovered in several regions in Southeast Asia, emphasising the need for alternative antimalarial medications such as doxorubicin, a potential IA [87 (opens in a new tab)]. Artemisinin and its derivatives exhibit antimicrobial activity against Gram-positive bacteria, Gram-negative bacteria, including Mycobacterium tuberculosis, Staphylococcus aureus, Escherichia coli, and Helicobacter pylori [88 (opens in a new tab)]. Artemisinin also displays an inhibitory effect on hepatitis C virus JFH-1 [89 (opens in a new tab)]. Last year, it was reported that artemisinin-based treatments display efficacy against SARS-CoV-2 in vitro, a contemporary demonstration of the potential of sesquiterpene lactones, and natural products in general, for pandemics [90 (opens in a new tab)].
The immunomodulatory activities of artemisinin and its derivatives on autoimmune diseases have been reviewed recently [91 (opens in a new tab)]. Sesquiterpene lactones have the capacity to regulate expressions of pro-inflammatory and anti-inflammatory cytokines, frequency and activation of T helper and B cells, and responsiveness of macrophages, DCs, neutrophils, mast cells, and MDSCs [92 (opens in a new tab)]. Consequently, artemisinin and its derivatives have a diverse application portfolio ranging from systemic lupus erythematosus (SLE) and multiple sclerosis to transplant rejection and cancer [[93] (opens in a new tab), [94] (opens in a new tab), [95] (opens in a new tab), [96] (opens in a new tab), [97] (opens in a new tab), [98] (opens in a new tab), [99] (opens in a new tab), [100] (opens in a new tab)]. The recent discovery of sesquiterpene lactones likely prefaces the characterisation of a broad-spectrum pharmacological profile in forthcoming years.
2.4. Fluoroquinolones
There is growing appreciation for the synergistic effect of artemisinin with fluoroquinolones for the treatment of malaria. Quinolone antibiotics are broad-spectrum bactericides that share a bicyclic core structure related to the substance 4-quinolone; addition of a fluorine atom at position C-6 has yielded fluoroquinolones, such as ciprofloxacin and moxifloxacin [101 (opens in a new tab)102 (opens in a new tab)]. Today, nearly all quinolone antibiotics in use are fluoroquinolones, and are used in human and veterinary medicine to treat bacterial infections, as well as in animal husbandry, particularly poultry production [103 (opens in a new tab)]. It has been understood since the 1990s that fluoroquinolones used for the treatment of bacterial infections exert activity against fungi, parasites, and viruses [[104] (opens in a new tab), [105] (opens in a new tab), [106] (opens in a new tab)]. That fluoroquinolones have been recommended for polymicrobial infections is simultaneously the recognition of the PPP of fluoroquinolones and a symptom of pre-COVID-19 thinking; the antimicrobial range of fluoroquinolones harbours significant untapped potential for pandemic-preparedness and bioterrorism-preparedness research i.e., preparing for a ‘monomicrobial’ disease by an unknown pathogen [107 (opens in a new tab)].
A demonstration of the heterogeneity of PPP, fluoroquinolones act as magic bullets against bacteria and parasites. With the former, fluoroquinolones inhibit two DNA topoisomerases essential for bacterial DNA synthesis and replication. Likewise, gyrase, a prokaryotic type II topoisomerase that serves the apicoplast genome (plDNA) of Plasmodium falciparum, is poisoned by fluoroquinolones which stabilise a catalytically inert ternary complex of enzyme, the plDNA substrate, and inhibitor; a mechanism perhaps responsible for the commercialisation of over 20 quinolones for malaria [108 (opens in a new tab)109 (opens in a new tab)]. Recently, several clinafloxacin-triazole hybrids presented antifungal activity against Candida albicans and Candida mycoderma [110 (opens in a new tab)]. Finally, an in silico study in 2020 showed that fluoroquinolones ciprofloxacin and moxifloxacin may inhibit SARS-CoV-2 replication by exhibiting stronger capacity for binding to its main protease than chloroquine and nelfinavir, a protease inhibitor antiretroviral drug [111 (opens in a new tab)].
Fluoroquinolones display multiple magic shield immunomodulatory actions leading to attenuation of the inflammatory response via inhibition of pro-inflammatory cytokines, albeit by unknown mechanisms and signal transduction pathways [112 (opens in a new tab)113 (opens in a new tab)]. It has also been demonstrated that, in analogy to chloroquine and tetracyclines, fluoroquinolones bind to and insert into cellular membranes, altering their fluidity [28 (opens in a new tab)114 (opens in a new tab)]. It would be interesting to compare the in vitro physicochemical interactions of these compounds with the lysosomotropic properties of the macrolide azithromycin, a broad-spectrum therapeutic. Indeed, both have been hypothesised to exert global physiological changes by altering pH [115 (opens in a new tab)116 (opens in a new tab)]. In addition to their use as first-line therapeutic agents for the management of severe community-acquired pneumonia, their favourable pharmacokinetics and safety profiles, and higher concentrations in the lungs in the case of levofloxacin and moxifloxacin, it has been proposed that respiratory fluoroquinolones be used in the treatment of SARS-CoV-2-associated pneumonia, furnishing this IA class with both magic bullet and magic shield pharmacology against COVID-19 [[117] (opens in a new tab), [118] (opens in a new tab), [119] (opens in a new tab)]. It is likely that the future of the fluoroquinolone class of IAs will comprise synthesis of an increasing array of hybrids and modifications, which in turn will reinforce the applicability of fluoroquinolones and their derivatives to many fields of medicine [[120] (opens in a new tab), [121] (opens in a new tab), [122] (opens in a new tab), [123] (opens in a new tab), [124] (opens in a new tab), [125] (opens in a new tab), [126] (opens in a new tab), [127] (opens in a new tab), [128] (opens in a new tab), [129] (opens in a new tab), [130] (opens in a new tab), [131] (opens in a new tab), [132] (opens in a new tab), [133] (opens in a new tab)].
2.5. Benzimidazoles
To combat AMR, many fluoroquinolones have been hybridised with benzimidazoles. Benzimidazole is a heterocyclic aromatic organic compound composed of benzene and imidazole [134 (opens in a new tab)]. The properties of benzimidazole and its derivatives have been studied for over a century and substituted benzimidazole derivatives have found applications in diverse therapeutic areas such as antiulcers, anticancer agents, and anthelmintics.
Antiparasitic effects of benzimidazoles are achieved by polypharmacological interference with sugar metabolism, alteration of energetic processes, and binding to tubulin to affect the cell cycle [135 (opens in a new tab)]. Many anthelmintic drugs such as albendazole, mebendazole, and triclabendazole also belong to the benzimidazole class of compounds [136 (opens in a new tab)]. Benzimidazole fungicides are commercialised, deriving their success by their magic bullet ability to bind fungal microtubules to inhibit hyphal growth [137 (opens in a new tab)]. Benzimidazoles also bind spindle microtubules to block nuclear division [138 (opens in a new tab)]. These cellular processes are also compromised in cancer and recent studies have indeed shown that benzimidazole derivatives exhibit prominent antineoplastic activity, further attesting to how the broad repositionability of IAs can also derive from their magic bullet properties [139 (opens in a new tab)]. Indeed, applications of benzimidazole-based compounds range from proton-pump inhibitors (antacids) to nitazenes (benzimidazole opioids). In the wake of COVID-19, benzimidazole-pyrazole hybrids are being synthesised with a view to address the dearth of suitable antiviral drugs [140 (opens in a new tab)141 (opens in a new tab)].
2.6. Macrolides
The quintessential antibiotics, it has long been accepted that macrolides exhibit a diverse range of properties with confirmed activity in prokaryotes and effects on inflammatory and immune cells, mucus secretion, and epithelial cell differentiation [142 (opens in a new tab)]. In fact, anti-inflammatory and immunomodulatory actions contribute to the therapeutic benefit of macrolides in most of the infectious disorders for which they are approved, as well as rationalising their application for other chronic inflammatory conditions that do not have primarily infectious aetiologies [143 (opens in a new tab)]. The chemical structures of certain macrolides are biomimetic, aiding their interactions with components of mammalian cells [144 (opens in a new tab)].
Macrolides constitute some of the most well-characterised magic bullets of the 20th century, including one of the most consequential antibiotics: erythromycin, which inhibits protein synthesis by binding 23 S rRNA in the 50 S subunit of ribosomes in susceptible bacteria [145 (opens in a new tab)]. Azithromycin, an erythromycin derivative, inhibits protein synthesis in the apicoplast of Plasmodium falciparum whilst blocking invasion of RBCs [146 (opens in a new tab)]. The antiparasitic ivermectin has been christened a ‘wonder drug’ due to its PPP [147 (opens in a new tab)]. Macrolides have been used in the treatment of HIV, herpes simplex type I, and influenza though this likely involves magic shield host-directed mechanisms [144 (opens in a new tab)]. That being said, amphotericin B boasts a feature on the WHO’s List of Essential Medicines for its ability to ameliorate systemic fungal infections; its magic bullet mechanism involves binding ergosterol leading to formation of pores in the fungal cell membrane, ion leakage, and ultimately fungal cell death [148 (opens in a new tab)].
The myriad magic shield properties of macrolides are still being elucidated. Atopic dermatitis and organ transplant rejection are addressed by immunosuppressant macrolide administration [149 (opens in a new tab)150 (opens in a new tab)]. Azithromycin-induced macrophage polarisation appears associated with alteration of STAT1 signalling through inhibition of NF-κB mediators [[151] (opens in a new tab), [152] (opens in a new tab), [153] (opens in a new tab), [154] (opens in a new tab)]. An improved understanding of the mechanisms associated with these agents could lead to promising therapeutic target discovery in a plethora of communicable and non-communicable immune disorders.
From the treatment of viral, bacterial, and fungal infections to the near-eradication of onchocerciasis, to supporting successful organ transplants, and to mitigating cancer, the applications of this IA class have had a profound impact on human health [[155] (opens in a new tab), [156] (opens in a new tab), [157] (opens in a new tab), [158] (opens in a new tab), [159] (opens in a new tab), [160] (opens in a new tab), [161] (opens in a new tab), [162] (opens in a new tab), [163] (opens in a new tab), [164] (opens in a new tab), [165] (opens in a new tab), [166] (opens in a new tab), [167] (opens in a new tab), [168] (opens in a new tab)]. My own discovery of IAs began with consolidating the PPP of azithromycin in 2020 during the first wave of the COVID-19 pandemic, and recent quantitative structure activity relationship (QSAR) studies provide new in silico and in vitro data pertaining to the ability of macrolides to impede entrance of SARS-CoV-2 into host cells [169 (opens in a new tab)170 (opens in a new tab)]. Macrolides are the prototypical IA class and as such buttress a benchmark against which other IA classes may be assessed.
2.7. Salicylanilides
Anthelmintic salicylanilides are amides of salicylic acid and aniline [171 (opens in a new tab)]. Owing their discovery to research for new antiseptics, salicylanilides have a variety of pharmacological uses: chlorinated derivatives, including niclosamide, oxyclozanide, and rafoxanide, are used as anthelmintics, especially as flukicides; and brominated derivatives, including dibromsalan, metabromsalan, and tribromsalan, are used as disinfectants with antibacterial and antifungal activities [172 (opens in a new tab)]. In a sharp albeit dangerous demonstration of the power of ideas, former President Trump stated ‘I see the disinfectant that knocks it out in a minute … is there a way we can do something like that by injection inside or almost a cleaning? It would be interesting to check that.’ [173 (opens in a new tab)174 (opens in a new tab)] By giving rise to both intravenous antimicrobials and surface disinfectants, the broad-range chemistry of salicylanilides is unironically a critical avenue for pandemic-preparedness research [175 (opens in a new tab)176 (opens in a new tab)].
Niclosamide and nitazoxanide are notable salicylanilides with clinical appraisals for a range of infectious diseases. Though it is unclear how they exert their antibacterial effects, their magic bullet antiparasitic mechanisms have begun to be delineated. As a hydrogen ionophore, niclosamide translocates protons across the inner membrane of mitochondria, resulting in the uncoupling of oxidative phosphorylation from electron transport and inhibiting the production of ATP. These effects are observed in isolated mitochondria of helminths and mammals. Selective toxicity is achieved by minimal systemic absorption combined with protective influence of protein binding. Niclosamide, an anthelmintic agent used to treat parasitic infections, also exhibits broad-spectrum antibacterial and broad-spectrum antiviral properties in vitro [177 (opens in a new tab)]. Nitazoxanide is a nitrothiazole derivative of salicylamide and is synthesised using the scaffold of niclosamide [178 (opens in a new tab)]. Studies of protozoa and anaerobic bacteria have shown that nitazoxanide is a magic bullet inhibitor of pyruvate-ferredoxin oxidoreductase (PFOR), an enzyme essential to anaerobic energy metabolism. However, interference with the PFOR enzyme-depending electron transfer reaction may not be the only pathway by which nitazoxanide exhibits antiprotozoal activity, and the mechanism of nitazoxanide’s activity against helminths is unknown.
It has been suggested that the broad activity of niclosamide is due to its magic shield immunomodulating activity [179 (opens in a new tab)180 (opens in a new tab)]. In 2012, niclosamide was discovered to be an entry inhibitor for a number of pH-dependent respiratory viruses, including influenza virus and human rhinoviruses [181 (opens in a new tab)]. Cell-biological and biochemical analyses and intracellular pH measurements have revealed that niclosamide neutralises acidic membrane-bounded compartments. Furthermore, niclosamide blocks rhinovirus infections synergistically with the macrolide proton ATPase inhibitor bafilomycin A1 [182 (opens in a new tab)]. Physico-chemical interference of host pathways is thus a leitmotif in IA pharmacology.
Though it is primarily used as an antiparasitic agent, nitazoxanide has been described as a ‘first-in-class broad-spectrum antiviral agent’ [183 (opens in a new tab)]. Indeed, much of its PPP stems from its ability to perturb the host immune landscape. First and second generation thiazolides upregulate gene expression of multiple components of the TLR- and type I IFN-signal transduction pathways, of multiple chemokines and cytokines, as well as production of IFNα by pDC, and that of IL2 and IFNγ by CD4+ T lymphocytes [184 (opens in a new tab)]. A double-blind, placebo-controlled clinical trial of patients with influenza infection showed a clear effect of nitazoxanide in reducing the severity of flu symptoms and viremia, and in increasing seroprotection and seroconversion rates [185 (opens in a new tab)186 (opens in a new tab)]. Moreover, immunomodulatory effects of thiazolides were stronger in FLU-stimulated cells compared to unstimulated control, suggesting that thiazolides reinforce host immune responses [187 (opens in a new tab)188 (opens in a new tab)]. It has been noted that this remarkable selectivity of thiazolides seems to explain the lack of adverse clinical side effects of nitazoxanide [189 (opens in a new tab)]. Nitazoxanide’s low cytotoxicity sets it apart from other immune-based therapies such as IFN, IL-2, and IL-12 that are associated with common and severe side effects resulting from generalised and extensive immune activation [190 (opens in a new tab)].
Due to their PPP, salicylanilides are preeminent IAs for pandemics, as evidenced by the ongoing campaign for their use against COVID-19 and monkeypox (also known as ‘mpox’) [[191] (opens in a new tab), [192] (opens in a new tab), [193] (opens in a new tab), [194] (opens in a new tab), [195] (opens in a new tab), [196] (opens in a new tab), [197] (opens in a new tab), [198] (opens in a new tab), [199] (opens in a new tab)]. Of particular note is that their immunomodulatory properties are better characterised than their magic bullet pharmacology. A transdisciplinary link with detergent chemistry adds further intrigue to the seventh IA class.
3. IA properties
Previously, I described how common disease networks within the host interactome constitute a consistency in the innate immune response in the presence of differing classes of pathogens [200 (opens in a new tab)]. Similarly, confluent chemical and pharmacological properties of IAs likely explain their PPP; in particular cationic amphiphilicity and lysosomotropicity, which are interestingly also found in therapeutics with high repositioning potential, even outside of infectious disease.
3.1. Lysosomotropicity and cationic amphiphilicity
Lysosomotropicity describes the ability of a therapeutic to accumulate within lysosomes and involves the rapid vacuolisation of the intracellular microenvironment by weakly basic amine compounds. These compounds are characterised by a hydrophobic aromatic ring or ring system coupled with a hydrophilic sidechain containing an ionisable amine functional group and are known as cationic amphiphilic drugs (CADs). Lysosomotropic compounds, much like amphiphilic antimicrobial peptides (AMPs) are not only used as antidepressants, antihistamines, antimicrobials, and antipsychotics, but potentially selectively destroy cancer cells [201 (opens in a new tab)]. Indeed, lysosomotropicity has been described as a way of therapeutically maintaining cellular homeostasis for acute maladies and, particularly with regard to COVID-19, may bridge the gap between antiviral and anti-inflammatory pharmacology [202 (opens in a new tab)].
In accordance with their lipophilicity, CADs diffuse through the membrane of acidic organelles in their unionised form and become protonated in the acidic lumen. Due to their decreased membrane permeability, protonated molecules cannot cross back to the cytosol and get trapped inside the acidic lumen where they accumulate. This ion trapping results in an increase in lysosome volume and impairing of their function, leading to downregulation of autophagy, reduction of endocytosis, and phospholipidosis due to reduction of phospholipid degradation. Phospholipidosis is the phenomenon whereby various lipid species accumulate inside the late endosomes and lysosomes. This phenotype is akin to that of patients with Niemann Pick type-C (NPC) disease, a lipid storage disorder [203 (opens in a new tab)]. If not too extreme, all these effects can be reversed upon cessation of treatment.
Evidence supporting antiviral activity of CADs has been well reviewed [[204] (opens in a new tab), [205] (opens in a new tab), [206] (opens in a new tab), [207] (opens in a new tab)]. It has also been anticipated that many drugs registered for non-antimicrobial use, due to their lysosomotropicity, exhibit intrinsic antiviral effects and constitute a pool of potential existing antivirals that may prove useful as the first line of defence in new viral outbreaks [208 (opens in a new tab)]. Two antiviral CADs have already been described as achieving their efficacy by lysosomotropicity: tilorone and umifenovir. Though the last 50 years have seen the use of tilorone as an interferon-inducing broad-spectrum antiviral, it is currently registered and used only in Russia and Ukraine for indications such as influenza, acute respiratory viral infection, viral hepatitis, viral encephalitis, and myelitis [209 (opens in a new tab)]. Its lysosomotropic potential has been described as comparable to chloroquine [210 (opens in a new tab)]. Umifenovir is registered in Russia and China for the treatment of influenza [211 (opens in a new tab)]. It is claimed to inhibit the membrane fusion of viruses with the endosomal membrane, which possibly occurs via increasing endosomal pH [212 (opens in a new tab)]. An open-label, randomised, clinical trial in Iran has reported umifenovir significantly contributes to improvements in peripheral oxygen saturation and duration of hospitalisation for COVID-19 patients [213 (opens in a new tab)]. Therefore, while lysosomotropicity is a magic bullet pharmacological property against some parasites, it is a broad-spectrum magic shield property against viruses.
Correlation of CAD-induced phospholipidosis with antiviral activity only accounts for part of the anti-infective pharmacology of a subset of IAs; while tetracyclines are not CADs, the immunomodulatory activity of macrolides appears to be linked with phospholipidosis. In LPS-stimulated J774A.1 cells, the extent of inhibition of pro-inflammatory markers IL-6 and PGE2 by macrolides significantly correlated with their extent of accumulation in cells, as well as with induction of phospholipidosis [214 (opens in a new tab)]. While recent reviews are debating on whether phospholipidosis is a true antiviral property or merely an in vitro artefact, phospholipidosis as a host-targeted mechanism common to different antimicrobial classes has potential to be a foundational principle of network PPP [215 (opens in a new tab)216 (opens in a new tab)].
3.2. Therapeutic range
As drug repositioning emerges as a cogent strategy for drug discovery, several studies will seek to delineate common properties of multi-purpose therapeutics (MPTs). MPTs can be defined as therapeutics which are repositioned according to more than one therapeutic class (analgesic, anticoagulant, anticancer, antidepressant, antidiabetic, antiepileptic, antimicrobial, antipsychotic, antipsychotic, antispasmodic, cardiovascular, depressant, sedative, stimulant). While many of these therapeutics are outside infectious disease research, the success of magic shields for treating infectious disease epitomises the need to include such host-directed drugs in antimicrobial research (Table 1 (opens in a new tab) ).
Table 1
Indications of MPTs. As underlying host-directed pharmacology of MPTs may share similarities with IA polypharmacology so MPTs listed here are potentially hitherto uncharacterised IAs suitable for infectious disease.
| Therapeutic | Original indication | Repositioned indication | Year | Pharmaceutical company |
|---|---|---|---|---|
| Amphotericin B | Fungal infection | Leishmaniasis | 1997 | NeXstar Pharma |
| Aspirin | Inflammation, pain | Antiplatelet, heart attack, stroke | Various | Various |
| Bromocriptine | Parkinson’s disease | Diabetes mellitus | 2009 | Novartis |
| Bupropion | Depression | Smoking cessation | 1997 | GSK |
| Colchicine | Gout | Recurrent pericarditis | 2009 | URL Pharma |
| Duloxetine | Depression | Stress urinary incontinence; fibromyalgia; chronic musculoskeletal pain | 2004; 2008; 2010 | Lilly; Lilly; Lilly |
| Eflornithine | Cancer | African sleeping sickness | 1990 | Aventis |
| Everolimus | Immunosuppressant | Cancer | Various | Novartis |
| Finasteride | Hypertension | Male pattern baldness | 1997 | Merck |
| Gabapentin | Epilepsy | Neuropathic pain | 2004 | Parke Davis |
| Methotrexate | Cancer | Psoriasis, rheumatoid arthritis | 2001 | Barr Labs |
| Miltefosine | Cancer | Visceral leishmaniasis | 2014 | Zentaris |
| Minoxidil | Hypertension | Male pattern baldness | 1988 | Upjohn |
| Propranolol | Hypertension | Migraine prophylaxis, tremors | Various | Various |
| Sildenafil | Angina | Erectile dysfunction | 1998 | Pfizer |
| Zidovudine | Cancer | HIV/AIDS | 1987 | Burroughs |
Open in a separate window (opens in a new tab)
One insightful study has revealed that MPTs are hallmarked by a higher hydrogen-bond donor count, suggesting a greater number of hydrogen bonds could contribute to the pluripotent drug-target binding mechanism across multiple disease phenotypes [217 (opens in a new tab)]. It is conceivable that lysosomotropic drugs with an optimum number of hydrogen bonds, by globally shifting cellular homeostasis away from the disease state (i.e. shifting the damage-response curve downwards), may be used for both communicable and non-communicable diseases without contributing to AMR (Fig. 2 (opens in a new tab) ). Therapeutics of the future may be furcated into acute and chronic classifications, where an indication is decided according to biomarker profiles across pathophysiology.
Properties of MPTs. Prospective properties range from pKa to polarisation of macrophages.
In conjunction with lysosomotropicity, disruption of mitochondrial function also appears to be a common denominator for MPTs, with psychotropic drugs, for example, showing anticancer activity by disrupting both mitochondrial and lysosomal function [218 (opens in a new tab)]. Similarly, antibiotics that target mitochondria effectively eradicate cancer stem cells across multiple tumour types. Mitochondrial biogenesis has been described as a global phenotypic characteristic highly conserved among cancer stem cells, enabling a mutation-independent approach to cancer therapy. 5 different classes of FDA-approved mitochondrially-targeted antibiotics include the erythromycins, tetracyclines, glycylcyclines, pyrvinium pamoate (an antiparasitic), and chloramphenicol. It has therefore been proposed that cancer can be treated like an infectious disease by repositioning FDA-approved antibiotics as preventative measures for anticancer therapy via eradication of cancer stem cells [219 (opens in a new tab)].
In closing, it is hoped that antimicrobial drugs of the future will be host-directed treatments that employ pharmacological mechanisms that ameliorate a range of non-communicable diseases, do not contribute to AMR, and ultimately antiquate traditional pathogen-killing antimicrobials.
4. IA development
Although IAs can be synthesised via traditional chemical and in silico methods of drug discovery (as with all small-molecule drugs), their PPP is only validated by repositioning. Following this, development of IAs for pandemics must involve 1) reducing their contributions to AMR and 2) increasing their therapeutic range. These can be achieved by chemical modification and validated by repositioning, both of which are accelerated by ever-evolving data-mining and machine learning (ML) processes which appraise chemical, pharmacological, and repositioning databases [220 (opens in a new tab)].
4.1. Chemical modification of existing antimicrobials
All small-molecule drugs used for infectious disease exhibit a conjectural bullet:shield ratio (BSR) which describes their pathogen-directed and host-modulating pharmacology. Reducing the bullet character of a given IA reduces its contributions to AMR [221 (opens in a new tab)]. Many IAs described in this review have already seen reduced BSRs by chemical modification; the archetype is the synthesis of non-antibiotic macrolides. In 2017, an azithromycin-based compound was found to reduce airway inflammation in chronic lung diseases whilst harbouring significantly diminished antimicrobial activity against a range of bacterial strains [222 (opens in a new tab)]. Moreover, the non-antibiotic macrolide EM900 inhibits rhinovirus infection and cytokine production in human airway epithelial cells [223 (opens in a new tab)].
Conjugation has also endowed existing antimicrobials with immunomodulatory activity. Influenza therapy with a single targeted compound is often limited in efficacy inasmuch as it contributes to AMR. However, uncontrolled release of virus-induced cytokines may contribute to high mortality of humans infected by H5N1 avian influenza virus. Therefore, novel dual-targeted bifunctional anti-influenza drugs were formed by conjugation with anti-inflammatory agents. The caffeic acid (CA)-bearing zanamivir (ZA) conjugates, ZA-7-CA (1) and ZA-7-CA-amide (7), showed simultaneous inhibition of influenza virus neuraminidase and suppression of pro-inflammatory cytokines [224 (opens in a new tab)]. These ZA conjugates provided protection of cells and mice against influenza infections. In fact, intranasal administration of low dosage (<1.2 μmol/kg/day) ZA conjugate exhibited much greater effect than the combination therapy with ZA and anti-inflammatory agents in protecting lethally-infected mice from H1N1 or N5N1 influenza viral infection. Conjugation to reduce BSR is a consolidative and promising area of research [225 (opens in a new tab)].
The BSR denotation for a given therapeutic is also dependent on the type of pathogen in consideration. The antibiotic azithromycin is a magic bullet for bacteria and malaria, but it is yet to be seen whether it behaves as a bullet across all parasite types; and azithromycin’s in vitro antiviral activity emerges from its host-directed lysosomotropicity [226 (opens in a new tab)]. Bullet:shield variability therefore exists across pathogen types and perhaps within a pathogen class [227 (opens in a new tab)]. Nevertheless, ‘shielding’, or chemical modification of IAs as a way to reduce BSR, can yield non-AMR-contributing therapeutics.
4.2. Repositioning existing antimicrobials and non-antimicrobials
While chemical modification changes the real BSR of a therapeutic, repositioning changes its perceived BSR. As an example, repositioning of the macrolide antiparasitic ivermectin for COVID-19 has unearthed its antiviral applicability and has raised questions as to how much of its antiparasitic pharmacology is determined by its pathogen-directed properties [228 (opens in a new tab)229 (opens in a new tab)].
Although repositioning of antimicrobials for non-communicable disease states have contributed to the acknowledgement of IAs, repositioning of non-antimicrobial drug classes towards infectious disease has also consolidated the potential of magic shields within the pathogenic context. Such shields have emerged from a variety of sources, from proton-pump inhibitors to antineoplastic agents [230 (opens in a new tab)]. Soon, antimicrobials that are crippled by their contributions to AMR, including IAs, may be replaced with those that exclusively exert network pharmacological effects on the host to achieve the same desired clinical outcome [231 (opens in a new tab)].
The molecular structures described in this review provide a starting point for drug-centric repositioning programmes which seek to discover non-AMR-inducing antimicrobials. Although a product of serendipity, there are 3 systematic approaches to drug repositioning: disease-centric, target-centric, and drug-centric [232 (opens in a new tab)]. Disease-centric approaches identify close relationships between an old and a new indication. A target-centric approach links a known target and its established drug to a new indication. Finally, a drug-centric approach connects a known drug to a new target and its associated indication. Despite the use of the umbrella term ‘drug’ repositioning, disease- and target-centric approaches have dominated the field; it has been suggested that the use of drug-centric approaches and structure-based techniques be exploited to realise the full potential of drug-target-disease connections. Analysis of repositioned drugs in an RDD database has revealed the majority of drugs have been redirected to the same disease family. This tendency was particularly pronounced within 2 categories of therapeutic indications: neoplasms and immune system disorders. These categories also have the highest number of repositioning cases in the database. Rapid repositioning approaches within the same disease family have been prioritised, leaving a pool of drug-target-disease connections unexplored [233 (opens in a new tab)]. The pleiotropic mechanism of action of IAs requires that IA-target-disease interactions be considered in the presence of a range of pathogen types.
While BSRs are a useful conceptual tool for understanding therapeutic contributions to AMR, they are confounded by the observation of the differential effect of a given therapeutic depending on its pathogen context. Azithromycin, for example, exhibits an altered immunomodulatory pharmacological landscape in the presence of pathogenic bacteria compared to viruses, furthering the need to consider a dynamic host-pathogen interactome model when screening therapeutic candidates and the need to recognise the importance of repositioning as a method for expanding our understanding of drug-disease networks [234 (opens in a new tab)].
5. Discussion
The term ‘IA’ sequesters a set of chemical compounds which harbour a pharmacological profile that is both unique and timely. The PPP of these compounds, which has not emerged from traditional magic bullet antimicrobial development and yet satisfies the need for host-directed, broad-spectrum antivirals, makes such therapeutics suitable for bioterrorism- and pandemic-preparedness research [235 (opens in a new tab)]. This broad pharmacology, likely emanating from their pKa and ability to alter intracellular pH, has also given rise to their applicability outside of infectious disease [236 (opens in a new tab)]. Indeed, by bridging the gap between unrelated disease types, IAs preface a therapeutic development paradigm beyond conventional nosology.
The rediscovery of existing antibiotics as anti-inflammatory agents is partly due to classical pharmacological approaches that have preceded modern target-based research. Classical pharmacology relies on phenotypic screening of chemical libraries of synthetic small molecules, natural products or extracts to identify substances that have a desirable therapeutic effect. The potency, selectivity, and other properties of these screening hits are optimised to produce candidate drugs. Only after the compounds have been discovered is an effort made to determine the biological target of the compounds through target validation experiments, often involving chemoproteomics. Since the 1990s, it has become popular to develop a hypothesis that a certain biological target is disease modifying and screen for compounds that modulate the activity of this purified target. Afterwards, these compounds are tested in animals to see if they have the desired effect; an approach known as ‘reverse pharmacology’ or target-based drug discovery [237 (opens in a new tab)]. However, recent statistical analyses revealed that a disproportionate number of first-in-class drugs with novel mechanisms of action emerge from phenotypic screening (classical pharmacology). The tendency to overestimate the ability of advances in basic research and brute-force screening methods to show a molecule as safe and effective in clinical trials has been described as a contributing factor to ‘Eroom’s law’ in drug discovery [238 (opens in a new tab)]. While this review does not present an argument for either approach, it is important to consider many IAs such as ivermectin have been discovered through phenotypic screening and use in animals prior to humans [239 (opens in a new tab)].
The identification of chemical and pharmacological commonalities across classes of IAs has significant implications for antimicrobial development. One emergent theme is lysosomotropicity, a property likely underpinning the concerted way in which IAs alter cellular homeostasis prior to and/or during infection [240 (opens in a new tab)241 (opens in a new tab)]. Last year, it was found that lysosomotropic agents including azithromycin, chloroquine, and hydroxychloroquine, can trigger the integrated stress response both in vitro and in vivo [242 (opens in a new tab)]. A link between lysosomotropicity and activation of the integrated stress response is perhaps one of many conserved, global mechanisms by which IAs achieve their PPP [243 (opens in a new tab)]. Further research will elucidate the links between lysosomotropicity and downstream network pharmacology.
The combinatorial use of IAs is another interesting avenue for further research. In one study over 20 years ago, nitazoxanide’s treatment of cryptosporidiosis, a parasitic infectious disease, was evaluated in an in vitro system in combination with azithromycin and rifabutin [244 (opens in a new tab)]. Good in vitro activity of the drug combinations was observed with safe cytotoxicity levels. In the ensuing years, increasing global significance of cryptosporidiosis among children has renewed efforts to improve control measures [245 (opens in a new tab)]. A gnotobiotic piglet model of acute diarrhoea was used to probe azithromycin/nitazoxanide against Cryptosporidium hominis, the species responsible for most human cases [246 (opens in a new tab)]. 10 day-treatment with recommended doses for children showed that treatment with azithromycin or nitazoxanide relieved symptoms early compared with untreated animals, while treatment with both azithromycin and nitazoxanide led to considerable symptomatic improvement and modest reduction of mucosal injury. More recently, Kelleni’s advocacy of azithromycin/nitazoxanide for COVID-19 has received significant academic attention [247 (opens in a new tab)248 (opens in a new tab)]. Yet, there are currently no studies investigating azithromycin/nitazoxanide for respiratory diseases. Combinations of IAs with magic shields, such as the combination of azithromycin and glucocorticoids for COVID-19, is a parallel line of enquiry for future research [249 (opens in a new tab)].
In June 2022, the World Health Organization declared the monkeypox outbreak an ‘evolving health threat’. While not a Public Health Emergency of International Concern (PHEIC), the most significant viral outbreak since COVID-19 warrants an investigation into its IA candidates. In this regard, salicylanilides have received particular attention since May of this year with South Korea’s Hyundai Bioscience’s announcement to submit a fast-track processing request to the FDA for the drug CP-COV03, whose active ingredient is niclosamide [250 (opens in a new tab)]. This followed research from Kansas State University which reported that niclosamide reduced vaccinia virus (another orthopoxvirus) proliferation to 1% at a concentration as low as 1 μM [251 (opens in a new tab)]. Hyundai Bioscience CEO Oh Sang Ki stated ‘CP-COV03 is a universal antiviral drug with niclosamide as the main ingredient, which can fight nearly all types of viruses. If CP-COV03 is approved as a treatment for monkeypox with the FDA’s fast-track designation, we will witness the birth of another innovative antiviral drug comparable to penicillin: the epitome of the 20th century’s wonder antibiotics.’ In December 2021, the company reported that CP-COV03 plus dexamethasone had been effective against severe COVID-19 patients, another clinical success for an IA/magic shield combinatory treatment regimen [252 (opens in a new tab)]. In 2018, the salicylanilide nitazoxanide was found to inhibit vaccinia virus replication at a viral lifecycle stage after entry but before late gene expression [253 (opens in a new tab)]. It has been hypothesised that this mechanism is likely due to nitazoxanide’s ability to interfere with metabolic adaptations needed for efficient virus replication, possibly by affecting acetyl-CoA production. The viruses now known to be sensitive to nitazoxanide include DNA and RNA viruses, viruses that replicate in the nucleus and in the cytoplasm, and enveloped and non-enveloped viruses. The extant application of traditionally antiparasitic therapeutics for monkeypox reaffirms the post-2020 epistemological shift from traditional magic bullet antivirals to host-modulating pan-pathogen pharmacological agents.
IAs are not the only class of antimicrobials that have challenged the magic bullet: magic shields can also be used to treat infectious disease, challenging previous denotations of the term ‘antimicrobial’. Decades of clinical investigations by van de Beek have cemented the administration of the anti-inflammatory agent dexamethasone for bacterial meningitis [254 (opens in a new tab)255 (opens in a new tab)]. During the COVID-19 pandemic, the same glucocorticoid was discovered to treat severe illness by reducing hyperinflammation [256 (opens in a new tab)]. The applicability of dexamethasone for both bacterial and viral diseases in the clinical setting is evidence of the pan-pathogen success of host-directed small-molecule therapy and warrants further repositioning studies to truly elucidate dexamethasone’s pan-pathogen potential. Unsurprisingly, as with IAs, dexamethasone is also used to treat cancers, including leukaemia and lymphoma [257 (opens in a new tab)]. It is important, therefore, to highlight both the pan-pathogen potential (and therefore pandemic-preparedness potential) and MPT potential of IAs and pure magic shield immunomodulators [258 (opens in a new tab)259 (opens in a new tab)].
Ultimately, this review propounds a pandemic-preparedness drug development paradigm centred around the phenomenon of PPP. It can be argued that there are two types of PPP: the first is magic bullet PPP, whereby a drug exhibits the ability to directly inhibit multiple pathogen classes by targeting conserved moieties within pathogen morphologies. This has been achieved by non-small-molecule therapeutic avenues, such as silver nanoparticles. However, such technologies are yet to be trialled clinically and are still far from being an affordable intervention for global health emergencies [260 (opens in a new tab)]. The second, magic shield PPP, is the ability to modulate the host immune system in order to benefit the host during any type of infection across multiple pathogen classes and is displayed by all immunomodulators and IAs. Although some IAs display magic bullet PPP, I maintain that all derive their PPP from their network pharmacological, immunomodulating properties (Fig. 3 (opens in a new tab) ) [[261] (opens in a new tab), [262] (opens in a new tab)].
Unification of four pillars of modern medicine: Pasteur’s germ theory, Béchamp’s terrain theory, Ehrlich’s magic bullet, and the magic shield. The magic bullet and the magic shield are not disparate concepts but two extremes of a continuum. All small-molecule drugs used to treat infectious diseases can be classified into 3 groups: antimicrobials, immunomodulators, and immunomodulating antimicrobials (IAs). This new model overcomes limitations of the magic bullet by recognising the polypharmacology of modern therapeutics and polymodality of the host target (indicated by gradients). As a result, the model predicts that A) Paragon magic shield immunomodulators such as dexamethasone can be used to treat infectious diseases such as COVID-19 and B) Both IAs and magic shields can be used against more than one pathogen class, giving rise to the phenomenon of pan-pathogen pharmacology (PPP). PPP is therefore a consequence of non-magic bullet antimicrobial development. Dotted lines indicate potential for shielding.
6. Conclusion
By the time a vaccine had been developed, over 200,000 people had died from COVID-19: a grim reminder of the need for therapeutic intervention for novel infectious diseases. Yet, more than antivirals, it was immunomodulators like dexamethasone which displayed clinical effectiveness against COVID-19. Therefore, while the magic shield model is an epistemological departure from a century-spanning paradigm of modern medicine, it recognises the pan-pathogen potential of IAs and immunomodulators, continually reinforced by coetaneous repositioning.
Availability of data and material
Not applicable.
Author contribution statement
Praveen Prathapan conceived, wrote, and edited the manuscript.
Code availability
Not applicable.
Ethics approval
Not applicable.
Funding statement
This research received no funding.
Declaration of competing interest
The author declare no known competing financial interests or personal relationships that could have appeared to influence the work reported in this paper.
Acknowledgements
Many thanks to my colleagues at the Department of Biochemistry and Trinity College, University of Oxford. My sincerest gratitude to Dr. Moro Balakrishnan from Bangalore, India for his insights on CADs and MPTs.
References
1. O’Grady J., Mwaba P., Zumla A. The health of prisoners. Lancet. 2011;377(9782):2001. doi: 10.1016/S0140-6736(11)60857-X. PMID: 21665029. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
2. Cavaillon J.M., Legout S. Louis Pasteur: between myth and reality. Biomolecules. 2022;12(4):596. doi: 10.3390/biom12040596. PMID: 35454184; PMCID: PMC9027159. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
3. Valent P., Groner B., Schumacher U., Superti-Furga G., Busslinger M., Kralovics R., Zielinski C., Penninger J.M., Kerjaschki D., Stingl G., Smolen J.S., Valenta R., Lassmann H., Kovar H., Jäger U., Kornek G., Müller M., Sörgel F. Paul Ehrlich (1854-1915) and his contributions to the foundation and birth of translational medicine. J. Innate. Immun. 2016;8(2):111–120. doi: 10.1159/000443526. PMID: 26845587; PMCID: PMC6738855. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
4. Zaffiri L., Gardner J., Toledo-Pereyra L.H. History of antibiotics. From salvarsan to cephalosporins. J. Invest. Surg. 2012;25(2):67–77. doi: 10.3109/08941939.2012.664099. PMID: 22439833. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
5. Thakur S., Mayank, Sarkar B., Ansari A.J., Khandelwal A., Arya A., Poduri R., Joshi G. Exploring the magic bullets to identify Achilles’ heel in SARS-CoV-2: delving deeper into the sea of possible therapeutic options in Covid-19 disease: an update. Food Chem. Toxicol. 2021;147 doi: 10.1016/j.fct.2020.111887. PMID: 33253764; PMCID: PMC7694479. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
6. Conly J.M., Johnston L.B. Coming full circle: from antibiotics to probiotics and prebiotics. Can. J. Infect Dis. Med. Microbiol. 2004;15(3):161–163. doi: 10.1155/2004/354909. PMID: 18159486; PMCID: PMC2094966. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
7. Muhaj F.F., George S.J., Nguyen C.D., Tyring S.K. Antimicrobials and resistance part II: antifungals, antivirals, and antiparasitics. J. Am. Acad. Dermatol. 2022;86(6):1207–1226. doi: 10.1016/j.jaad.2021.11.065. PMID: 35122895. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
8. Allegrante J.P., Auld M.E., Natarajan S. Preventing COVID-19 and its sequela: “there is No magic bullet… It’s just behaviors. Am. J. Prev. Med. 2020;59(2):288–292. doi: 10.1016/j.amepre.2020.05.004. PMID: 32591282; PMCID: PMC7260531. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
9. Kozlov M. Merck’s COVID pill loses its lustre: what that means for the pandemic. Nature. 2021 doi: 10.1038/d41586-021-03667-0. PMID: 34903873. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
10. Wiener S.L. Strategies of biowarfare defense. Mil. Med. 1987;152(1):25–28. PMID: 3103005. [PubMed (opens in a new tab)] [Google Scholar (opens in a new tab)]
11. Biodefense Strategic Plan NIH: national institute of allergy and infectious diseases. 2007. www.niaid.nih.gov (opens in a new tab)
12. Horby P., Lim W.S., Emberson J.R., Mafham M., Bell J.L., Linsell L., Staplin N., Brightling C., Ustianowski A., Elmahi E., Prudon B., Green C., Felton T., Chadwick D., Rege K., Fegan C., Chappell L.C., Faust S.N., Jaki T., Jeffery K., Montgomery A., Rowan K., Juszczak E., Baillie J.K., Haynes R., Landray M.J., RECOVERY Collaborative Group Dexamethasone in hospitalized patients with covid-19. N. Engl. J. Med. 2021;384(8):693–704. doi: 10.1056/NEJMoa2021436. PMID: 32678530; PMCID: PMC7383595. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
13. Firth A., Prathapan P. Azithromycin: the first broad-spectrum therapeutic. Eur. J. Med. Chem. 2020;207 doi: 10.1016/j.ejmech.2020.112739. PMID: 32871342; PMCID: PMC7434625. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
14. Pirofski L.A., Casadevall A. The damage-response framework as a tool for the physician-scientist to understand the pathogenesis of infectious diseases. J. Infect. Dis. 2018;218(suppl_1):S7–S11. doi: 10.1093/infdis/jiy083. PMID: 30124977; PMCID: PMC6093430. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
15. Ho T.T., Tran Q.T., Chai C.L. The polypharmacology of natural products. Future Med. Chem. 2018;10(11):1361–1368. doi: 10.4155/fmc-2017-0294. PMID: 29673257. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
16. Crielaard B.J., Lammers T., Schiffelers R.M., Storm G. Drug targeting systems for inflammatory disease: one for all, all for one. J. Contr. Release. 2012;161(2):225–234. doi: 10.1016/j.jconrel.2011.12.014. PMID: 22226771. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
17. Machado E.R., Carlos D., Sorgi C.A., Ramos S.G., Souza D.I., Soares E.G., Costa-Cruz J.M., Ueta M.T., Aronoff D.M., Faccioli L.H. Dexamethasone effects in the Strongyloides venezuelensis infection in a murine model. Am. J. Trop. Med. Hyg. 2011;84(6):957–966. doi: 10.4269/ajtmh.2011.10-0490. PMID: 21633034; PMCID: PMC3110371. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
18. Griffin M.O., Fricovsky E., Ceballos G., Villarreal F. Tetracyclines: a pleitropic family of compounds with promising therapeutic properties. Review of the literature. Am. J. Physiol. Cell Physiol. 2010;299(3):C539–C548. doi: 10.1152/ajpcell.00047.2010. PMID: 20592239; PMCID: PMC2944325. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
19. Guo Z. The modification of natural products for medical use. Acta Pharm. Sin. B. 2017;7(2):119–136. doi: 10.1016/j.apsb.2016.06.003. PMID: 28303218; PMCID: PMC5343118. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
20. Chopra I., Roberts M. Tetracycline antibiotics: mode of action, applications, molecular biology, and epidemiology of bacterial resistance. Microbiol. Mol. Biol. Rev. 2001;65(2):232–260. doi: 10.1128/MMBR.65.2.232-260.2001. second page, table of contents. PMID: 11381101; PMCID: PMC99026. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
21. Zhang W., Ames B.D., Tsai S.C., Tang Y. Engineered biosynthesis of a novel amidated polyketide, using the malonamyl-specific initiation module from the oxytetracycline polyketide synthase. Appl. Environ. Microbiol. 2006;72(4):2573–2580. doi: 10.1128/AEM.72.4.2573-2580.2006. PMID: 16597959; PMCID: PMC1449064. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
22. Zhou S., Shao Y., Gao N., Zhu S., Ma Y., Deng J. Chlorination and chloramination of tetracycline antibiotics: disinfection by-products formation and influential factors. Ecotoxicol. Environ. Saf. 2014;107:30–35. doi: 10.1016/j.ecoenv.2014.05.008. PMID: 24905694. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
23. Shastri R.A., Krishnaswamy K. Undernutrition and tetracycline half life. Clin. Chim. Acta. 1976;66(2):157–164. doi: 10.1016/0009-8981(76)90052-8. PMID: 1245065. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
24. Jahantigh M., Samadi K., Dizaji R.E., Salari S. Antimicrobial resistance and prevalence of tetracycline resistance genes in Escherichia coli isolated from lesions of colibacillosis in broiler chickens in Sistan, Iran. BMC Vet. Res. 2020;16(1):267. doi: 10.1186/s12917-020-02488-z. PMID: 32746815; PMCID: PMC7397602. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
25. Grossman T.H. Tetracycline antibiotics and resistance. Cold Spring Harb Perspect Med. 2016;6(4):a025387. doi: 10.1101/cshperspect.a025387. PMID: 26989065; PMCID: PMC4817740. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
26. Batool Z., Lomakin I.B., Polikanov Y.S., Bunick C.G. Sarecycline interferes with tRNA accommodation and tethers mRNA to the 70S ribosome. Proc. Natl. Acad. Sci. U. S. A. 2020;117(34):20530–20537. doi: 10.1073/pnas.2008671117. PMID: 32817463; PMCID: PMC7456112. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
27. Chukwudi C.U. rRNA binding sites and the molecular mechanism of action of the tetracyclines. Antimicrob. Agents Chemother. 2016;60(8):4433–4441. doi: 10.1128/AAC.00594-16. PMID: 27246781; PMCID: PMC4958212. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
28. Delcour A.H. Outer membrane permeability and antibiotic resistance. Biochim. Biophys. Acta. 2009;1794(5):808–816. doi: 10.1016/j.bbapap.2008.11.005. PMID: 19100346; PMCID: PMC2696358. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
29. Dahl E.L., Shock J.L., Shenai B.R., Gut J., DeRisi J.L., Rosenthal P.J. Tetracyclines specifically target the apicoplast of the malaria parasite Plasmodium falciparum. Antimicrob. Agents Chemother. 2006;50(9):3124–3131. doi: 10.1128/AAC.00394-06. PMID: 16940111; PMCID: PMC1563505. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
30. O’Shea K.L., Singh N.D. Tetracycline-exposed Drosophila melanogaster males produce fewer offspring but a relative excess of sons. Ecol. Evol. 2015;5(15):3130–3139. doi: 10.1002/ece3.1535. PMID: 26357541; PMCID: PMC4559055. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
31. Garrido-Mesa N., Zarzuelo A., Gálvez J. Minocycline: far beyond an antibiotic. Br. J. Pharmacol. 2013;169(2):337–352. doi: 10.1111/bph.12139. PMID: 23441623; PMCID: PMC3651660. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
32. Zhang H., Mao C., Li J., Huang Z., Gu X., Shen X., Ding H. Pharmacokinetic/Pharmacodynamic integration of doxycycline against Mycoplasma hyopneumoniae in an in vitro model. Front. Pharmacol. 2019;10:1088. doi: 10.3389/fphar.2019.01088. PMID: 31620004; PMCID: PMC6763577. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
33. Bode C., Diedrich B., Muenster S., Hentschel V., Weisheit C., Rommelsheim K., Hoeft A., Meyer R., Boehm O., Knuefermann P., Baumgarten G. Antibiotics regulate the immune response in both presence and absence of lipopolysaccharide through modulation of Toll-like receptors, cytokine production and phagocytosis in vitro. Int. Immunopharm. 2014;18(1):27–34. doi: 10.1016/j.intimp.2013.10.025. PMID: 24239744. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
34. Pang T., Wang J., Benicky J., Saavedra J.M. Minocycline ameliorates LPS-induced inflammation in human monocytes by novel mechanisms including LOX-1, Nur 77 and LITAF inhibition. Biochim. Biophys. Acta. 2012;1820(4):503–510. doi: 10.1016/j.bbagen.2012.01.011. PMID: 22306153; PMCID: PMC3307860. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
35. Krady J.K., Basu A., Allen C.M., Xu Y., LaNoue K.F., Gardner T.W., Levison S.W. Minocycline reduces proinflammatory cytokine expression, microglial activation, and caspase-3 activation in a rodent model of diabetic retinopathy. Diabetes. 2005;54(5):1559–1565. doi: 10.2337/diabetes.54.5.1559. PMID: 15855346. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
36. Ketelut-Carneiro N., Silva G.K., Rocha F.A., Milanezi C.M., Cavalcanti-Neto F.F., Zamboni D.S., Silva J.S. IL-18 triggered by the Nlrp3 inflammasome induces host innate resistance in a pulmonary model of fungal infection. J. Immunol. 2015;194(9):4507–4517. doi: 10.4049/jimmunol.1402321. PMID: 25825440. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
37. Hamarsheh S., Zeiser R. NLRP3 inflammasome activation in cancer: a double-edged sword. Front. Immunol. 2020;11:1444. doi: 10.3389/fimmu.2020.01444. PMID: 32733479; PMCID: PMC7360837. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
38. Missiroli S., Perrone M., Boncompagni C., Borghi C., Campagnaro A., Marchetti F., Anania G., Greco P., Fiorica F., Pinton P., Giorgi C. Targeting the NLRP3 inflammasome as a new therapeutic option for overcoming cancer. Cancers. 2021;13(10):2297. doi: 10.3390/cancers13102297. PMID: 34064909; PMCID: PMC8151587. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
39. Alsaadi M., Tezcan G., Garanina E.E., Hamza S., McIntyre A., Rizvanov A.A., Khaiboullina S.F. Doxycycline attenuates cancer cell growth by suppressing NLRP3-mediated inflammation. Pharmaceuticals. 2021;14(9):852. doi: 10.3390/ph14090852. PMID: 34577552; PMCID: PMC8466018. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
40. Zhang L., Xu L., Zhang F., Vlashi E. Doxycycline inhibits the cancer stem cell phenotype and epithelial-to-mesenchymal transition in breast cancer. Cell Cycle. 2017;16(8):737–745. doi: 10.1080/15384101.2016.1241929. PMID: 27753527; PMCID: PMC5405729. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
41. Zhao C., Zhao W. NLRP3 inflammasome-A key player in antiviral responses. Front. Immunol. 2020;11:211. doi: 10.3389/fimmu.2020.00211. PMID: 32133002; PMCID: PMC7040071. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
42. Negrette A. Encefalitis epidémica. Invest. Clin. 1960;1:13–34. [Google Scholar (opens in a new tab)]
43. Francini E., Miano S.T., Fiaschi A.I., Francini G. Doxycycline or minocycline may be a viable treatment option against SARS-CoV-2. Med. Hypotheses. 2020;144 doi: 10.1016/j.mehy.2020.110054. PMID: 32758890; PMCID: PMC7320853. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
44. Gironi L.C., Damiani G., Zavattaro E., Pacifico A., Santus P., Pigatto P.D.M., Cremona O., Savoia P. Tetracyclines in COVID-19 patients quarantined at home: literature evidence supporting real-world data from a multicenter observational study targeting inflammatory and infectious dermatoses. Dermatol. Ther. 2021;34(1) doi: 10.1111/dth.14694. PMID: 33354849; PMCID: PMC7883087. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
45. Negrette A. Tetraciclina y SIDA [tetracycline and AIDS] Invest. Clin. 1990;31(3):117–119. Spanish. PMID: 2101639. [PubMed (opens in a new tab)] [Google Scholar (opens in a new tab)]
46. Negrette A. Tetraciclina y virus pequeños. Editorial. Invest. Clin. 1980;21:235–238. [Google Scholar (opens in a new tab)]
47. Zakeri B., Wright G.D. Chemical biology of tetracycline antibiotics. Biochem. Cell. Biol. 2008;86(2):124–136. doi: 10.1139/O08-002. PMID: 18443626. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
48. Humar A., McGilvray I., Phillips M.J., Levy G.A. Severe acute respiratory syndrome and the liver. Hepatology. 2004;39(2):291–294. doi: 10.1002/hep.20069. PMID: 14767979; PMCID: PMC7165921. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
49. Rothan H.A., Mohamed Z., Paydar M., Rahman N.A., Yusof R. Inhibitory effect of doxycycline against dengue virus replication in vitro. Arch. Virol. 2014;159(4):711–718. doi: 10.1007/s00705-013-1880-7. PMID: 24142271. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
50. Ohe M., Furuya K., Goudarzi H. Tetracycline plus macrolide: a potential therapeutic regimen for COVID-19? Biosci Trends. 2021;14(6):467–468. doi: 10.5582/bst.2020.03443. PMID: 33390423. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
51. Huo Z., Gridnev I.D., Yamamoto Y. A method for the synthesis of substituted quinolines via electrophilic cyclization of 1-azido-2-(2-propynyl)benzene. J. Org. Chem. 2010;75(4):1266–1270. doi: 10.1021/jo902603v. PMID: 20099928. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
52. Chen Y.L., Chen I.L., Wang T.C., Han C.H., Tzeng C.C. Synthesis and anticancer evaluation of certain 4-anilinofuro[2,3-b]quinoline and 4-anilinofuro[3,2-c]quinoline derivatives. Eur. J. Med. Chem. 2005;40(9):928–934. doi: 10.1016/j.ejmech.2005.04.003. PMID: 15913847. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
53. Foley M., Tilley L. Quinoline antimalarials: mechanisms of action and resistance and prospects for new agents. Pharmacol. Ther. 1998;79(1):55–87. doi: 10.1016/s0163-7258(98)00012-6. PMID: 9719345. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
54. Ibáñez de Garayo M., Liu W., Rondeau N.C., Damoci C.B., Miranda J.J.L. Rationally repurposed nitroxoline inhibits preclinical models of Epstein-Barr virus-associated lymphoproliferation. J. Antibiot. (Tokyo) 2021;74(10):763–766. doi: 10.1038/s41429-021-00433-2. PMID: 34163027; PMCID: PMC8472899. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
55. Raphemot R., Posfai D., Derbyshire E.R. Current therapies and future possibilities for drug development against liver-stage malaria. J. Clin. Invest. 2016;126(6):2013–2020. doi: 10.1172/JCI82981. PMID: 27249674; PMCID: PMC4887158. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
56. de Pina-Costa A., Silvino A.C.R., Dos Santos E.M., Pedro R.S., Moreira J., Umana G.L., da Silva A.D.T., da Rosa Santos O.H.L., de Deus Henriques K.M., Daniel-Ribeiro C.T., Brasil P., Sousa T.N., Siqueira A.M. Increased primaquine total dose prevents Plasmodium vivax relapses in patients with impaired CYP2D6 activity: report of three cases. Malar. J. 2021;20(1):341. doi: 10.1186/s12936-021-03869-x. PMID: 34391426; PMCID: PMC8364036. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
57. Schaer C.A., Laczko E., Schoedon G., Schaer D.J., Vallelian F. Chloroquine interference with hemoglobin endocytic trafficking suppresses adaptive heme and iron homeostasis in macrophages: the paradox of an antimalarial agent. Oxid. Med. Cell. Longev. 2013;2013 doi: 10.1155/2013/870472. PMID: 23840921; PMCID: PMC3693174. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
58. Senerovic L., Opsenica D., Moric I., Aleksic I., Spasić M., Vasiljevic B. Quinolines and quinolones as antibacterial, antifungal, anti-virulence, antiviral and anti-parasitic agents. Adv. Exp. Med. Biol. 2020;1282:37–69. doi: 10.1007/5584_2019_428. PMID: 31515709. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
59. Tzouvelekis A., Karampitsakos T., Bouros D. The role of hydroxychloroquine in coronavirus disease 2019. A versatile tool at the service of humanity. Front. Med. 2020;7:176. doi: 10.3389/fmed.2020.00176. PMID: 32391370; PMCID: PMC7193980. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
60. Chandler L.C., Yusuf I.H., McClements M.E., Barnard A.R., MacLaren R.E., Xue K. Immunomodulatory effects of hydroxychloroquine and chloroquine in viral infections and their potential application in retinal gene therapy. Int. J. Mol. Sci. 2020;21(14):4972. doi: 10.3390/ijms21144972. PMID: 32674481; PMCID: PMC7404262. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
61. An J., Woodward J.J., Sasaki T., Minie M., Elkon K.B. Cutting edge: antimalarial drugs inhibit IFN-β production through blockade of cyclic GMP-AMP synthase-DNA interaction. J. Immunol. 2015;194(9):4089–4093. doi: 10.4049/jimmunol.1402793. PMID: 25821216. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
62. Allen M.E., Golding A., Rus V., Karabin N.B., Li S., Lescott C.J., Bobbala S., Scott E.A., Szeto G.L. Targeted delivery of chloroquine to antigen-presenting cells enhances inhibition of the type I interferon response. ACS Biomater. Sci. Eng. 2021;7(12):5666–5677. doi: 10.1021/acsbiomaterials.1c01047. PMID: 34813288. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
63. Gies V., Bekaddour N., Dieudonné Y., Guffroy A., Frenger Q., Gros F., Rodero M.P., Herbeuval J.P., Korganow A.S. Beyond anti-viral effects of chloroquine/hydroxychloroquine. Front. Immunol. 2020;11:1409. doi: 10.3389/fimmu.2020.01409. PMID: 32714335; PMCID: PMC7343769. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
64. Yao X., Ye F., Zhang M., Cui C., Huang B., Niu P., Liu X., Zhao L., Dong E., Song C., Zhan S., Lu R., Li H., Tan W., Liu D. Vitro antiviral activity and projection of optimized dosing design of hydroxychloroquine for the treatment of severe acute respiratory syndrome coronavirus 2 (SARS-CoV-2) Clin. Infect. Dis. 2020;71(15):732–739. doi: 10.1093/cid/ciaa237. PMID: 32150618; PMCID: PMC7108130. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
65. Lauria A., La Monica G., Bono A., Martorana A. Quinoline anticancer agents active on DNA and DNA-interacting proteins: from classical to emerging therapeutic targets. Eur. J. Med. Chem. 2021;220 doi: 10.1016/j.ejmech.2021.113555. PMID: 34052677. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
66. Fiorillo M., Lamb R., Tanowitz H.B., Mutti L., Krstic-Demonacos M., Cappello A.R., Martinez-Outschoorn U.E., Sotgia F., Lisanti M.P. Repurposing atovaquone: targeting mitochondrial complex III and OXPHOS to eradicate cancer stem cells. Oncotarget. 2016;7(23):34084–34099. doi: 10.18632/oncotarget.9122. PMID: 27136895; PMCID: PMC5085139. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
67. Wallace D.C. Mitochondria and cancer. Nat. Rev. Cancer. 2012;12(10):685–698. doi: 10.1038/nrc3365. PMID: 23001348; PMCID: PMC4371788. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
68. Nayak A.P., Kapur A., Barroilhet L., Patankar M.S. Oxidative phosphorylation: a target for novel therapeutic strategies against ovarian cancer. Cancers. 2018;10(9):337. doi: 10.3390/cancers10090337. PMID: 30231564; PMCID: PMC6162441. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
69. Muz B., de la Puente P., Azab F., Azab A.K. The role of hypoxia in cancer progression, angiogenesis, metastasis, and resistance to therapy. Hypoxia. 2015;3:83–92. doi: 10.2147/HP.S93413. PMID: 27774485; PMCID: PMC5045092. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
70. Ming L., Cheng K., Chen Y., Yang R., Chen D. Enhancement of tumor lethality of ROS in photodynamic therapy. Cancer Med. 2021;10(1):257–268. doi: 10.1002/cam4.3592. PMID: 33141513; PMCID: PMC7826450. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
71. Li X., Kwon N., Guo T., Liu Z., Yoon J. Innovative strategies for hypoxic-tumor photodynamic therapy. Angew Chem. Int. Ed. Engl. 2018;57(36):11522–11531. doi: 10.1002/anie.201805138. PMID: 29808948. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
72. Ashton T.M., Fokas E., Kunz-Schughart L.A., Folkes L.K., Anbalagan S., Huether M., Kelly C.J., Pirovano G., Buffa F.M., Hammond E.M., Stratford M., Muschel R.J., Higgins G.S., McKenna W.G. The anti-malarial atovaquone increases radiosensitivity by alleviating tumour hypoxia. Nat. Commun. 2016;7 doi: 10.1038/ncomms12308. PMID: 27453292; PMCID: PMC4962491. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
73. Selim M.R., Zahran M.A., Belal A., Abusaif M.S., Shedid S.A., Mehany A.B.M., Elhagali G.A.M., Ammar Y.A. Hybridized quinoline derivatives as anticancer agents: design, synthesis, biological evaluation and molecular docking. Anti Cancer Agents Med. Chem. 2019;19(4):439–452. doi: 10.2174/1871520618666181112121058. PMID: 30417798. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
74. Li Y.Q., Zheng Z., Liu Q.X., Lu X., Zhou D., Zhang J., Zheng H., Dai J.G. Repositioning of antiparasitic drugs for tumor treatment. Front. Oncol. 2021;11 doi: 10.3389/fonc.2021.670804. PMID: 33996598; PMCID: PMC8117216. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
75. Xu J., Cole D.C., Chang C.P., Ayyad R., Asselin M., Hao W., Gibbons J., Jelinsky S.A., Saraf K.A., Park K. Inhibition of the signal transducer and activator of transcription-3 (STAT3) signaling pathway by 4-oxo-1-phenyl-1,4-dihydroquinoline-3-carboxylic acid esters. J. Med. Chem. 2008;51(14):4115–4121. doi: 10.1021/jm701271y. PMID: 18578470. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
76. Belayneh A. Off-label use of chloroquine and hydroxychloroquine for COVID-19 treatment in africa against WHO recommendation. Res. Rep. Trop. Med. 2020;11:61–72. doi: 10.2147/RRTM.S269936. PMID: 32982538; PMCID: PMC7505701. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
77. Dima A., Jurcut C., Chasset F., Felten R., Arnaud L. Hydroxychloroquine in systemic lupus erythematosus: overview of current knowledge, Ther. Adv. Musculoskelet. Dis. 2022;14 doi: 10.1177/1759720X211073001. PMID: 35186126; PMCID: PMC8848057. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
78. Domizio J.D., Gulen M.F., Saidoune F., Thacker V.V., Yatim A., Sharma K., Nass T., Guenova E., Schaller M., Conrad C., Goepfert C., de Leval L., Garnier C.V., Berezowska S., Dubois A., Gilliet M., Ablasser A. The cGAS-STING pathway drives type I IFN immunopathology in COVID-19. Nature. 2022;603(7899):145–151. doi: 10.1038/s41586-022-04421-w. PMID: 35045565; PMCID: PMC8891013. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
79. Insuasty D., Vidal O., Bernal A., Marquez E., Guzman J., Insuasty B., Quiroga J., Svetaz L., Zacchino S., Puerto G., Abonia R. Antimicrobial activity of quinoline-based hydroxyimidazolium hybrids. Antibiotics (Basel) 2019;8(4):239. doi: 10.3390/antibiotics8040239. PMID: 31795101; PMCID: PMC6963836. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
80. Teng P., Li C., Peng Z., Anne Marie V., Nimmagadda A., Su M., Li Y., Sun X., Cai J. Facilely accessible quinoline derivatives as potent antibacterial agents. Bioorg. Med. Chem. 2018;26(12):3573–3579. doi: 10.1016/j.bmc.2018.05.031. PMID: 29858158; PMCID: PMC6084461. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
81. Kaur P., Anuradha, Chandra A., Tanwar T., Sahu S.K., Mittal A. Emerging quinoline- and quinolone-based antibiotics in the light of epidemics. Chem. Biol. Drug Des. 2022 doi: 10.1111/cbdd.14025. PMID: 35128812. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
82. Chadwick M., Trewin H., Gawthrop F., Wagstaff C. Sesquiterpenoids lactones: benefits to plants and people. Int. J. Mol. Sci. 2013;14(6):12780–12805. doi: 10.3390/ijms140612780. PMID: 23783276; PMCID: PMC3709812. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
83. Ivanescu B., Miron A., Corciova A. Sesquiterpene lactones from Artemisia genus: biological activities and methods of analysis. J. Anal. Methods Chem. 2015;2015 doi: 10.1155/2015/247685. PMID: 26495156; PMCID: PMC4606394. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
84. Su X.Z., Miller L.H. The discovery of artemisinin and the Nobel prize in Physiology or medicine. Sci. China Life Sci. 2015;58(11):1175–1179. doi: 10.1007/s11427-015-4948-7. PMID: 26481135; PMCID: PMC4966551. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
85. Nosten F., White N.J. Artemisinin-based combination treatment of falciparum malaria. Am. J. Trop. Med. Hyg. 2007;77(6 Suppl):181–192. PMID: 18165491. [PubMed (opens in a new tab)] [Google Scholar (opens in a new tab)]
86. Tsamesidis I., Pério P., Pantaleo A., Reybier K. Oxidation of erythrocytes enhance the production of reactive species in the presence of artemisinins. Int. J. Mol. Sci. 2020;21(13):4799. doi: 10.3390/ijms21134799. PMID: 32646002; PMCID: PMC7369783. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
87. Rosenthal P.J. Has artemisinin resistance emerged in Africa? Lancet Infect. Dis. 2021;21(8):1056–1057. doi: 10.1016/S1473-3099(21)00168-7. PMID: 33864802. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
88. Appalasamy S., Lo K.Y., Ch’ng S.J., Nornadia K., Othman A.S., Chan L.K. Antimicrobial activity of artemisinin and precursor derived from in vitro plantlets of Artemisia annua L. BioMed Res. Int. 2014;2014 doi: 10.1155/2014/215872. PMID: 24575401; PMCID: PMC3915762. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
89. Obeid S., Alen J., Nguyen V.H., Pham V.C., Meuleman P., Pannecouque C., Le T.N., Neyts J., Dehaen W., Paeshuyse J. Artemisinin analogues as potent inhibitors of in vitro hepatitis C virus replication. PLoS One. 2013;8(12) doi: 10.1371/journal.pone.0081783. PMID: 24349127; PMCID: PMC3859510. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
90. Zhou Y., Gilmore K., Ramirez S., Settels E., Gammeltoft K.A., Pham L.V., Fahnøe U., Feng S., Offersgaard A., Trimpert J., Bukh J., Osterrieder K., Gottwein J.M., Seeberger P.H. In vitro efficacy of artemisinin-based treatments against SARS-CoV-2. Sci. Rep. 2021;11(1) doi: 10.1038/s41598-021-93361-y. PMID: 34272426; PMCID: PMC8285423. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
91. Qiu F., Liu J., Mo X., Liu H., Chen Y., Dai Z. Immunoregulation by artemisinin and its derivatives: a new role for old antimalarial drugs. Front. Immunol. 2021;12 doi: 10.3389/fimmu.2021.751772. PMID: 34567013; PMCID: PMC8458561. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
92. Li D., Qi J., Wang J., Pan Y., Li J., Xia X., Dou H., Hou Y. Protective effect of dihydroartemisinin in inhibiting senescence of myeloid-derived suppressor cells from lupus mice via Nrf 2/HO-1 pathway. Free Radic. Biol. Med. 2019;143:260–274. doi: 10.1016/j.freeradbiomed.2019.08.013. PMID: 31419476. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
93. Dong J., Chen Y., Yang W., Zhang X., Li L. Antitumor and anti-angiogenic effects of artemisinin on breast tumor xenografts in nude mice. Res. Vet. Sci. 2020;129:66–69. doi: 10.1016/j.rvsc.2020.01.005. PMID: 31945670. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
94. Krishna S., Bustamante L., Haynes R.K., Staines H.M. Artemisinins: their growing importance in medicine. Trends Pharmacol. Sci. 2008;29(10):520–527. doi: 10.1016/j.tips.2008.07.004. PMID: 18752857; PMCID: PMC2758403. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
95. Nagelschmitz J., Voith B., Wensing G., Roemer A., Fugmann B., Haynes R.K., Kotecka B.M., Rieckmann K.H., Edstein M.D. First assessment in humans of the safety, tolerability, pharmacokinetics, and ex vivo pharmacodynamic antimalarial activity of the new artemisinin derivative artemisone. Antimicrob. Agents Chemother. 2008;52(9):3085–3091. doi: 10.1128/AAC.01585-07. PMID: 18559649; PMCID: PMC2533467. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
96. Navaratnam V., Mansor S.M., Sit N.W., Grace J., Li Q., Olliaro P. Pharmacokinetics of artemisinin-type compounds. Clin. Pharmacokinet. 2000;39(4):255–270. doi: 10.2165/00003088-200039040-00002. PMID: 11069212. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
97. Blanco E., Shen H., Ferrari M. Principles of nanoparticle design for overcoming biological barriers to drug delivery. Nat. Biotechnol. 2015;33(9):941–951. doi: 10.1038/nbt.3330. PMID: 26348965; PMCID: PMC4978509. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
98. Zhang Z.Y., Yu S.Q., Miao L.Y., Huang X.Y., Zhang X.P., Zhu Y.P., Xia X.H., Li D.Q. [Artesunate combined with vinorelbine plus cisplatin in treatment of advanced non-small cell lung cancer: a randomized controlled trial] Zhong Xi Yi Jie He Xue Bao. 2008;6(2):134–138. doi: 10.3736/jcim20080206. Chinese. PMID: 18241646. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
99. Matos M.S., Anastácio J.D., Nunes Dos Santos C. Sesquiterpene lactones: promising natural compounds to fight inflammation. Pharmaceutics. 2021;13(7):991. doi: 10.3390/pharmaceutics13070991. PMID: 34208907; PMCID: PMC8309091. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
100. Arberas-Jiménez I., Rizo-Liendo A., Nocchi N., Sifaoui I., Chao-Pellicer J., Souto M.L., Suárez-Gómez B., Díaz-Marrero A.R., Fernández J.J., Piñero J.E., Lorenzo-Morales J. Sesquiterpene lactones as potential therapeutic agents against Naegleria fowleri. Biomed. Pharmacother. 2022;147 doi: 10.1016/j.biopha.2022.112694. PMID: 35131659. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
101. Pham T.D.M., Ziora Z.M., Blaskovich M.A.T. Quinolone antibiotics. Medchemcomm. 2019;10(10):1719–1739. doi: 10.1039/c9md00120d. PMID: 31803393; PMCID: PMC6836748. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
102. Kocsis B., Domokos J., Szabo D. Chemical structure and pharmacokinetics of novel quinolone agents represented by avarofloxacin, delafloxacin, finafloxacin, zabofloxacin and nemonoxacin. Ann. Clin. Microbiol. Antimicrob. 2016;15(1):34. doi: 10.1186/s12941-016-0150-4. PMID: 27215369; PMCID: PMC4878067. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
103. Price L.B., Lackey L.G., Vailes R., Silbergeld E. The persistence of fluoroquinolone-resistant Campylobacter in poultry production. Environ. Health Perspect. 2007;115(7):1035–1039. doi: 10.1289/ehp.10050. PMID: 17637919; PMCID: PMC1913601. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
104. Lode H., Borner K., Koeppe P. Pharmacodynamics of fluoroquinolones. Clin. Infect. Dis. 1998;27(1):33–39. doi: 10.1086/514623. PMID: 9675446. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
105. Khan A.A., Araujo F.G., Brighty K.E., Gootz T.D., Remington J.S. Anti-Toxoplasma gondii activities and structure-activity relationships of novel fluoroquinolones related to trovafloxacin. Antimicrob. Agents Chemother. 1999;43(7):1783–1787. doi: 10.1128/AAC.43.7.1783. PMID: 10390245; PMCID: PMC89366. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
106. Furet Y.X., Pechère J.C. Newly documented antimicrobial activity of quinolones. Eur. J. Clin. Microbiol. Infect. Dis. 1991;10(4):249–254. doi: 10.1007/BF01966997. PMID: 1864284. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
107. Shams W.E., Evans M.E. Guide to selection of fluoroquinolones in patients with lower respiratory tract infections. Drugs. 2005;65(7):949–991. doi: 10.2165/00003495-200565070-00004. PMID: 15892589; PMCID: PMC7100689. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
108. Tang Girdwood S.C., Nenortas E., Shapiro T.A. Targeting the gyrase of Plasmodium falciparum with topoisomerase poisons. Biochem. Pharmacol. 2015;95(4):227–237. doi: 10.1016/j.bcp.2015.03.018. PMID: 25881748; PMCID: PMC4449814. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
109. Millanao A.R., Mora A.Y., Villagra N.A., Bucarey S.A., Hidalgo A.A. Biological effects of quinolones: a family of broad-spectrum antimicrobial agents. Molecules. 2021;26(23):7153. doi: 10.3390/molecules26237153. PMID: 34885734; PMCID: PMC8658791. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
110. Wang Y., Damu G.L., Lv J.S., Geng R.X., Yang D.C., Zhou C.H. Design, synthesis and evaluation of clinafloxacin triazole hybrids as a new type of antibacterial and antifungal agents. Bioorg. Med. Chem. Lett. 2012;22(17):5363–5366. doi: 10.1016/j.bmcl.2012.07.064. PMID: 22884108. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
111. Marciniec K., Beberok A., Pęcak P., Boryczka S., Wrześniok D. Ciprofloxacin and moxifloxacin could interact with SARS-CoV-2 protease: preliminary in silico analysis. Pharmacol. Rep. 2020;72(6):1553–1561. doi: 10.1007/s43440-020-00169-0. PMID: 33063271; PMCID: PMC7561236. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
112. Zusso M., Lunardi V., Franceschini D., Pagetta A., Lo R., Stifani S., Frigo A.C., Giusti P., Moro S. Ciprofloxacin and levofloxacin attenuate microglia inflammatory response via TLR4/NF-kB pathway. J. Neuroinflammation. 2019;16(1):148. doi: 10.1186/s12974-019-1538-9. PMID: 31319868; PMCID: PMC6637517. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
113. Dalhoff A. Antiviral, antifungal, and antiparasitic activities of fluoroquinolones optimized for treatment of bacterial infections: a puzzling paradox or a logical consequence of their mode of action? Eur. J. Clin. Microbiol. Infect. Dis. 2015;34(4):661–668. doi: 10.1007/s10096-014-2296-3. PMID: 25515946; PMCID: PMC7087824. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
114. Gombos I., Vígh L. Membrane fluidity in the center of fever-enhanced immunity. Cell Cycle. 2015;14(19):3014–3015. doi: 10.1080/15384101.2015.1069506. PMID: 26207859; PMCID: PMC4825518. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
115. PRINCIPLE Trial Collaborative Group Azithromycin for community treatment of suspected COVID-19 in people at increased risk of an adverse clinical course in the UK (PRINCIPLE): a randomised, controlled, open-label, adaptive platform trial. Lancet. 2021;397(10279):1063–1074. doi: 10.1016/S0140-6736(21)00461-X. PMID: 33676597; PMCID: PMC7972318. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
116. Smith C.B., Evavold C., Kersh G.J. The effect of pH on antibiotic efficacy against coxiella burnetii in axenic media. Sci. Rep. 2019;9(1) doi: 10.1038/s41598-019-54556-6. PMID: 31792307; PMCID: PMC6889355. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
117. Albertson T.E., Dean N.C., El Solh A.A., Gotfried M.H., Kaplan C., Niederman M.S. Fluoroquinolones in the management of community-acquired pneumonia. Int. J. Clin. Pract. 2010;64(3):378–388. doi: 10.1111/j.1742-1241.2009.02239.x. PMID: 20456176. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
118. Vardakas K.Z., Siempos, Grammatikos A., Athanassa Z., Korbila I.P., Falagas M.E. Respiratory fluoroquinolones for the treatment of community-acquired pneumonia: a meta-analysis of randomized controlled trials. CMAJ (Can. Med. Assoc. J.) 2008;179(12):1269–1277. doi: 10.1503/cmaj.080358. Erratum in: CMAJ. 2009 Jan 6;180(1):79. PMID: 19047608; PMCID: PMC2585120. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
119. Karampela I., Dalamaga M. Could respiratory fluoroquinolones, levofloxacin and moxifloxacin, prove to be beneficial as an adjunct treatment in COVID-19? Arch. Med. Res. 2020;51(7):741–742. doi: 10.1016/j.arcmed.2020.06.004. PMID: 32546446; PMCID: PMC7275144. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
120. Robertson G.T., Bonventre E.J., Doyle T.B., Du Q., Duncan L., Morris T.W., Roche E.D., Yan D., Lynch A.S. In vitro evaluation of CBR-2092, a novel rifamycin-quinolone hybrid antibiotic: microbiology profiling studies with staphylococci and streptococci. Antimicrob. Agents Chemother. 2008;52(7):2324–2334. doi: 10.1128/AAC.01651-07. PMID: 18443106; PMCID: PMC2443883. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
121. Fedorowicz J., Saczewski J. Modifications of quinolones and fluoroquinolones: hybrid compounds and dual-action molecules. Monatsh. Chem. 2018;149(7):1199–1245. doi: 10.1007/s00706-018-2215-x. PMID: 29983452; PMCID: PMC6006264. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
122. Yadav V., Talwar P. Repositioning of fluoroquinolones from antibiotic to anti-cancer agents: an underestimated truth. Biomed. Pharmacother. 2019;111:934–946. doi: 10.1016/j.biopha.2018.12.119. PMID: 30841473. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
123. Uivarosi V. Metal complexes of quinolone antibiotics and their applications: an update. Molecules. 2013;18(9):11153–11197. doi: 10.3390/molecules180911153. PMID: 24029748; PMCID: PMC6269848. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
124. Măciucă A.M., Munteanu A.C., Uivarosi V. Quinolone complexes with lanthanide ions: an insight into their analytical applications and biological activity. Molecules. 2020;25(6):1347. doi: 10.3390/molecules25061347. PMID: 32188087; PMCID: PMC7144119. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
125. Aranha O., Grignon R., Fernandes N., McDonnell T.J., Wood D.P., Jr., Sarkar F.H. Suppression of human prostate cancer cell growth by ciprofloxacin is associated with cell cycle arrest and apoptosis. Int. J. Oncol. 2003;22(4):787–794. PMID: 12632069. [PubMed (opens in a new tab)] [Google Scholar (opens in a new tab)]
126. Yadav V., Varshney P., Sultana S., Yadav J., Saini N. Moxifloxacin and ciprofloxacin induces S-phase arrest and augments apoptotic effects of cisplatin in human pancreatic cancer cells via ERK activation. BMC Cancer. 2015;15:581. doi: 10.1186/s12885-015-1560-y. PMID: 26260159; PMCID: PMC4531397. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
127. Sousa E., Graça I., Baptista T., Vieira F.Q., Palmeira C., Henrique R., Jerónimo C. Enoxacin inhibits growth of prostate cancer cells and effectively restores microRNA processing. Epigenetics. 2013;8(5):548–558. doi: 10.4161/epi.24519. PMID: 23644875; PMCID: PMC3741225. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
128. Rizk J.G., Kalantar-Zadeh K., Mehra M.R., Lavie C.J., Rizk Y., Forthal D.N. Pharmaco-immunomodulatory therapy in COVID-19. Drugs. 2020;80(13):1267–1292. doi: 10.1007/s40265-020-01367-z. PMID: 32696108; PMCID: PMC7372203. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
129. Armstrong A., Reddy R., Chadha D., Kircik L. Supplement article: a novel drug delivery method: retrometabolic drug design. J. Drugs Dermatol. JDD. 2022;21(4):s5–s10. PMID: 35389593. [PubMed (opens in a new tab)] [Google Scholar (opens in a new tab)]
130. Gao F., Zhang X., Wang T., Xiao J. Quinolone hybrids and their anti-cancer activities: an overview. Eur. J. Med. Chem. 2019;165:59–79. doi: 10.1016/j.ejmech.2019.01.017. PMID: 30660827. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
131. Lindamulage I.K., Vu H.Y., Karthikeyan C., Knockleby J., Lee Y.F., Trivedi P., Lee H. Novel quinolone chalcones targeting colchicine-binding pocket kill multidrug-resistant cancer cells by inhibiting tubulin activity and MRP1 function. Sci. Rep. 2017;7(1) doi: 10.1038/s41598-017-10972-0. PMID: 28860494; PMCID: PMC5578999. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
132. Fiorito J., Saeed F., Zhang H., Staniszewski A., Feng Y., Francis Y.I., Rao S., Thakkar D.M., Deng S.X., Landry D.W., Arancio O. Synthesis of quinoline derivatives: discovery of a potent and selective phosphodiesterase 5 inhibitor for the treatment of Alzheimer’s disease. Eur. J. Med. Chem. 2013;60:285–294. doi: 10.1016/j.ejmech.2012.12.009. PMID: 23313637; PMCID: PMC3582828. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
133. Vuong H., Stentzel M.R., Klumpp D.A. Superacid-promoted synthesis of quinoline derivatives. Tetrahedron Lett. 2020;61(12) doi: 10.1016/j.tetlet.2020.151630. PMID: 33299258; PMCID: PMC7720793. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
134. Ates-Alagoz Z. Antimicrobial activities of 1-H-Benzimidazole-based molecules. Curr. Top. Med. Chem. 2016;16(26):2953–2962. doi: 10.2174/1568026616666160506130226. PMID: 27150377. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
135. Mook R.A., Jr., Ren X.R., Wang J., Piao H., Barak L.S., Kim Lyerly H., Chen W. Benzimidazole inhibitors from the Niclosamide chemotype inhibit Wnt/β-catenin signaling with selectivity over effects on ATP homeostasis. Bioorg. Med. Chem. 2017;25(6):1804–1816. doi: 10.1016/j.bmc.2017.01.046. PMID: 28233680; PMCID: PMC5490664. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
136. Alvarez L., Moreno G., Moreno L., Ceballos L., Shaw L., Fairweather I., Lanusse C. Comparative assessment of albendazole and triclabendazole ovicidal activity on Fasciola hepatica eggs. Vet. Parasitol. 2009;164(2–4):211–216. doi: 10.1016/j.vetpar.2009.05.014. PMID: 19560276. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
137. Ahuja R., Sidhu A., Bala A., Arora D., Sharma P. 2020. Structure Based Approach for Twin-Enzyme Targeted Benzimidazolyl-1,2,4-Triazole Molecular Hybrids as Antifungal Agents; pp. 5832–5848. 13(6) [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
138. Minagawa M., Shirato M., Toya M., Sato M. Dual impact of a benzimidazole resistant β-tubulin on microtubule behavior in fission yeast. Cells. 2021;10(5):1042. doi: 10.3390/cells10051042. PMID: 33925026; PMCID: PMC8145593. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
139. Yadav S., Narasimhan B., Kaur H. Perspectives of benzimidazole derivatives as anticancer agents in the new era. Anti Cancer Agents Med. Chem. 2016;16(11):1403–1425. doi: 10.2174/1871520616666151103113412. PMID: 26526461. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
140. Marinescu M. Synthesis of antimicrobial benzimidazole-pyrazole compounds and their biological activities. Antibiotics (Basel) 2021;10(8):1002. doi: 10.3390/antibiotics10081002. PMID: 34439052; PMCID: PMC8389006. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
141. Oprea T.I., Overington J.P. Computational and practical aspects of drug repositioning. Assay Drug Dev. Technol. 2015;13(6):299–306. doi: 10.1089/adt.2015.29011.tiodrrr. PMID: 26241209; PMCID: PMC4533090. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
142. Kricker J.A., Page C.P., Gardarsson F.R., Baldursson O., Gudjonsson T., Parnham M.J. Nonantimicrobial actions of macrolides: overview and perspectives for future development. Pharmacol. Rev. 2021;73(4):233–262. doi: 10.1124/pharmrev.121.000300. PMID: 34716226. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
143. Zarogoulidis P., Papanas N., Kioumis I., Chatzaki E., Maltezos E., Zarogoulidis K. Macrolides: from in vitro anti-inflammatory and immunomodulatory properties to clinical practice in respiratory diseases. Eur. J. Clin. Pharmacol. 2012;68(5):479–503. doi: 10.1007/s00228-011-1161-x. PMID: 22105373. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
144. Lenz K.D., Klosterman K.E., Mukundan H., Kubicek-Sutherland J.Z. Macrolides: from toxins to therapeutics. Toxins. 2021;13(5):347. doi: 10.3390/toxins13050347. PMID: 34065929; PMCID: PMC8150546. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
145. Jelić D., Antolović R. From erythromycin to azithromycin and new potential ribosome-binding antimicrobials. Antibiotics (Basel) 2016;5(3):29. doi: 10.3390/antibiotics5030029. PMID: 27598215; PMCID: PMC5039525. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
146. Muralidharan V., Striepen B. Teaching old drugs new tricks to stop malaria invasion in its tracks. BMC Biol. 2015;13:72. doi: 10.1186/s12915-015-0185-6. PMID: 26349580; PMCID: PMC4563855. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
147. Crump A., Ōmura S. Ivermectin, ‘wonder drug’ from Japan: the human use perspective. Proc. Jpn. Acad. Ser. B Phys. Biol. Sci. 2011;87(2):13–28. doi: 10.2183/pjab.87.13. PMID: 21321478; PMCID: PMC3043740. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
148. Kneale M., Bartholomew J.S., Davies E., Denning D.W. Global access to antifungal therapy and its variable cost. J. Antimicrob. Chemother. 2016;71(12):3599–3606. doi: 10.1093/jac/dkw325. PMID: 27516477. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
149. Marsland A.M., Griffiths C.E. Therapeutic potential of macrolide immunosuppressants in dermatology. Expet Opin. Invest. Drugs. 2004;13(2):125–137. doi: 10.1517/13543784.13.2.125. PMID: 14996647. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
150. Poshekhontseva V.Y., Fokina V.V., Tarlachkov S.V., Machulin A.V., Shutov A.A., Donova M.V. Streptomyces tsukubensis VKM aс-2618d-an effective producer of tacrolimus. Appl. Biochem. Microbiol. 2021;57(9):939–948. doi: 10.1134/S0003683821090064. PMID: 34924587; PMCID: PMC8670718. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
151. Haydar D., Cory T.J., Birket S.E., Murphy B.S., Pennypacker K.R., Sinai A.P., Feola D.J. Azithromycin polarizes macrophages to an M2 phenotype via inhibition of the STAT1 and NF-κB signaling pathways. J. Immunol. 2019;203(4):1021–1030. doi: 10.4049/jimmunol.1801228. PMID: 31263039; PMCID: PMC6684391. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
152. Vrančić M., Banjanac M., Nujić K., Bosnar M., Murati T., Munić V., Stupin Polančec D., Belamarić D., Parnham M.J., Eraković Haber V. Azithromycin distinctively modulates classical activation of human monocytes in vitro. Br. J. Pharmacol. 2012;165(5):1348–1360. doi: 10.1111/j.1476-5381.2011.01576.x. PMID: 21726210; PMCID: PMC3372721. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
153. Zhang B., Kopper T.J., Liu X., Cui Z., Van Lanen S.G., Gensel J.C. Macrolide derivatives reduce proinflammatory macrophage activation and macrophage-mediated neurotoxicity. CNS Neurosci. Ther. 2019;25(5):591–600. doi: 10.1111/cns.13092. PMID: 30677254; PMCID: PMC6488883. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
154. Zhang B., Bailey W.M., Kopper T.J., Orr M.B., Feola D.J., Gensel J.C. Azithromycin drives alternative macrophage activation and improves recovery and tissue sparing in contusion spinal cord injury. J. Neuroinflammation. 2015;12:218. doi: 10.1186/s12974-015-0440-3. PMID: 26597676; PMCID: PMC4657208. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
155. Qiao X., Wang X., Shang Y., Li Y., Chen S.Z. Azithromycin enhances anticancer activity of TRAIL by inhibiting autophagy and up-regulating the protein levels of DR4/5 in colon cancer cells in vitro and in vivo. Cancer Commun. 2018;38(1):43. doi: 10.1186/s40880-018-0309-9. PMID: 29970185; PMCID: PMC6029027. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
156. Kanoh S., Rubin B.K. Mechanisms of action and clinical application of macrolides as immunomodulatory medications. Clin. Microbiol. Rev. 2010;23(3):590–615. doi: 10.1128/CMR.00078-09. PMID: 20610825; PMCID: PMC2901655. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
157. Zhang P., Zhang Y., Liu K., Liu B., Xu W., Gao J., Ding L., Tao L. Ivermectin induces cell cycle arrest and apoptosis of HeLa cells via mitochondrial pathway. Cell Prolif. 2019;52(2) doi: 10.1111/cpr.12543. PMID: 30515909; PMCID: PMC6496724. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
158. Dou Q., Chen H.N., Wang K., Yuan K., Lei Y., Li K., Lan J., Chen Y., Huang Z., Xie N., Zhang L., Xiang R., Nice E.C., Wei Y., Huang C. Ivermectin induces cytostatic autophagy by blocking the PAK1/akt Axis in breast cancer. Cancer Res. 2016;76(15):4457–4469. doi: 10.1158/0008-5472.CAN-15-2887. PMID: 27302166. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
159. Wang K., Gao W., Dou Q., Chen H., Li Q., Nice E.C., Huang C. Ivermectin induces PAK1-mediated cytostatic autophagy in breast cancer. Autophagy. 2016;12(12):2498–2499. doi: 10.1080/15548627.2016.1231494. PMID: 27657889; PMCID: PMC5173258. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
160. Dominguez-Gomez G., Chavez-Blanco A., Medina-Franco J.L., Saldivar-Gonzalez F., Flores-Torrontegui Y., Juarez M., Díaz-Chávez J., Gonzalez-Fierro A., Dueñas-González A. Ivermectin as an inhibitor of cancer stem-like cells. Mol. Med. Rep. 2018;17(2):3397–3403. doi: 10.3892/mmr.2017.8231. PMID: 29257278. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
161. Gao A., Liang H., Wang X., Zhang X., Jing M., Zhang J., Yan Y., Xiang W. Reversal effects of two new milbemycin compounds on multidrug resistance in MCF-7/adr cells in vitro. Eur. J. Pharmacol. 2011;659(2–3):108–113. doi: 10.1016/j.ejphar.2011.03.023. PMID: 21458446. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
162. Xiang W., Gao A., Liang H., Li C., Gao J., Wang Q., Shuang B., Zhang J., Yan Y., Wang X. Reversal of P-glycoprotein-mediated multidrug resistance in vitro by milbemycin compounds in adriamycin-resistant human breast carcinoma (MCF-7/adr) cells. Toxicol. Vitro. 2010;24(6):1474–1481. doi: 10.1016/j.tiv.2010.07.020. PMID: 20656007. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
163. Low Z.Y., Farouk I.A., Lal S.K. Drug repositioning: new approaches and future prospects for life-debilitating diseases and the COVID-19 pandemic outbreak. Viruses. 2020;12(9):1058. doi: 10.3390/v12091058. PMID: 32972027; PMCID: PMC7551028. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
164. Kim H.S. Drug repositioning: exploring new indications for existing drug-disease relationships. Endocrinol Metab (Seoul) 2022;37(1):62–64. doi: 10.3803/EnM.2022.1403. PMID: 35255602; PMCID: PMC8901967. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
165. Peigneur S., Tytgat J. Toxins in drug discovery and pharmacology. Toxins. 2018;10(3):126. doi: 10.3390/toxins10030126. PMID: 29547537; PMCID: PMC5869414. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
166. Espiña B., Rubiolo J.A. Marine toxins and the cytoskeleton: pectenotoxins, unusual macrolides that disrupt actin. FEBS J. 2008;275(24):6082–6088. doi: 10.1111/j.1742-4658.2008.06714.x. PMID: 19016860. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
167. Jimeno A. Eribulin: rediscovering tubulin as an anticancer target. Clin. Cancer Res. 2009;15(12):3903–3905. doi: 10.1158/1078-0432.CCR-09-1023. PMID: 19509144. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
168. Swami U., Shah U., Goel S. Eribulin in cancer treatment. Mar. Drugs. 2015;13(8):5016–5058. doi: 10.3390/md13085016. PMID: 26262627; PMCID: PMC4557013. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
169. Kruger D., Prathapan P. Azithromycin: the first broad-spectrum therapeutic. J. Transl. Autoimmun. 2020 doi: 10.1016/j.jtauto.2020.100062. PMID: 32839756; PMCID: PMC7439010. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
170. Galvez J., Zanni R., Galvez-Llompart M., Benlloch J.M. Macrolides may prevent severe acute respiratory syndrome coronavirus 2 entry into cells: a quantitative structure activity relationship study and experimental validation. J. Chem. Inf. Model. 2021;61(4):2016–2025. doi: 10.1021/acs.jcim.0c01394. PMID: 33734704; PMCID: PMC7986980. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
171. Swan G.E. The pharmacology of halogenated salicylanilides and their anthelmintic use in animals. J. S. Afr. Vet. Assoc. 1999;70(2):61–70. doi: 10.4102/jsava.v70i2.756. PMID: 10855824. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
172. McCullough F.S., Gayral P., Duncan J., Christie J.D. Molluscicides in schistosomiasis control. Bull. World Health Organ. 1980;58(5):681–689. PMID: 6975179; PMCID: PMC2395986. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [Google Scholar (opens in a new tab)]
173. Kiely E., Farley R. The white house spins trump’s disinfectant remarks. https://www.factcheck.org/2020/04/the-white-house-spins-trumps-disinfectant-remarks/ (opens in a new tab) Online.
174. Clark D. Trump suggests ‘injection’ of disinfectant to beat coronavirus and ‘clean’ the lungs. https://www.nbcnews.com/politics/donald-trump/trump-suggests-injection-disinfectant-beat-coronavirus-clean-lungs-n1191216 (opens in a new tab) Online.
175. Krátký M., Vinšová J. Antiviral activity of substituted salicylanilides—a review. Mini Rev. Med. Chem. 2011;11(11):956–967. doi: 10.2174/138955711797068382. PMID: 21762100. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
176. Blake S., Shaabani N., Eubanks L.M., Maruyama J., Manning J.T., Beutler N., Paessler S., Ji H., Teijaro J.R., Janda K.D. Salicylanilides reduce SARS-CoV-2 replication and suppress induction of inflammatory cytokines in a rodent model. ACS Infect. Dis. 2021;7(8):2229–2237. doi: 10.1021/acsinfecdis.1c00253. PMID: 34339171; PMCID: PMC8353890. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
177. Xu J., Shi P.Y., Li H., Zhou J. Broad spectrum antiviral agent niclosamide and its therapeutic potential. ACS Infect. Dis. 2020;6(5):909–915. doi: 10.1021/acsinfecdis.0c00052. PMID: 32125140; PMCID: PMC7098069. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
178. Stachulski A.V., Taujanskas J., Pate S.L., Rajoli R.K.R., Aljayyoussi G., Pennington S.H., Ward S.A., Hong W.D., Biagini G.A., Owen A., Nixon G.L., Leung S.C., O’Neill P.M. Therapeutic potential of nitazoxanide: an appropriate choice for repurposing versus SARS-CoV-2? ACS Infect. Dis. 2021;7(6):1317–1331. doi: 10.1021/acsinfecdis.0c00478. PMID: 33352056; PMCID: PMC7771247. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
179. Wu C.S., Li Y.R., Chen J.J., Chen Y.C., Chu C.L., Pan I.H., Wu Y.S., Lin C.C. Antihelminthic niclosamide modulates dendritic cells activation and function. Cell. Immunol. 2014;288(1–2):15–23. doi: 10.1016/j.cellimm.2013.12.006. PMID: 24561310; PMCID: PMC7094312. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
180. Jang S.G., Lee J., Hong S.M., Song Y.S., Kim M.J., Kwok S.K., Cho M.L., Park S.H. Niclosamide suppresses the expansion of follicular helper T cells and alleviates disease severity in two murine models of lupus via STAT3. J. Transl. Med. 2021;19(1):86. doi: 10.1186/s12967-021-02760-2. PMID: 33632240; PMCID: PMC7908700. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
181. Jurgeit A., McDowell R., Moese S., Meldrum E., Schwendener R., Greber U.F. Niclosamide is a proton carrier and targets acidic endosomes with broad antiviral effects. PLoS Pathog. 2012;8(10) doi: 10.1371/journal.ppat.1002976. PMID: 23133371; PMCID: PMC3486884. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
182. Murer L., Petkidis A., Vallet T., Vignuzzi M., Greber U.F. Chemical evolution of rhinovirus identifies capsid-destabilizing mutations driving low-pH-independent genome uncoating. J. Virol. 2022;96(2) doi: 10.1128/JVI.01060-21. PMID: 34705560; PMCID: PMC8791267. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
183. Rossignol J.F. Nitazoxanide: a first-in-class broad-spectrum antiviral agent. Antivir. Res. 2014;110:94–103. doi: 10.1016/j.antiviral.2014.07.014. PMID: 25108173; PMCID: PMC7113776. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
184. Trabattoni D., Gnudi F., Ibba S.V., Saulle I., Agostini S., Masetti M., Biasin M., Rossignol J.F., Clerici M. Thiazolides elicit anti-viral innate immunity and reduce HIV replication. Sci. Rep. 2016;6 doi: 10.1038/srep27148. PMID: 27250526; PMCID: PMC4890011. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
185. Gnudi Federica. 2014. IMMUNOMODULATORY EFFECTS OF NITAZOXANIDE AND RELATED MOLECULES. [Google Scholar (opens in a new tab)]
186. Haffizulla J., Hartman A., Hoppers M., Resnick H., Samudrala S., Ginocchio C., Bardin M., Rossignol J.F., US Nitazoxanide Influenza Clinical Study Group Effect of nitazoxanide in adults and adolescents with acute uncomplicated influenza: a double-blind, randomised, placebo-controlled, phase 2b/3 trial. Lancet Infect. Dis. 2014;14(7):609–618. doi: 10.1016/S1473-3099(14)70717-0. PMID: 24852376; PMCID: PMC7164783. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
187. Casadevall A., Pirofski L.A. Host-pathogen interactions: basic concepts of microbial commensalism, colonization, infection, and disease. Infect. Immun. 2000;68(12):6511–6518. doi: 10.1128/IAI.68.12.6511-6518.2000. PMID: 11083759; PMCID: PMC97744. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
188. Casadevall A., Pirofski L.A. Microbiology: ditch the term pathogen. Nature. 2014;516(7530):165–166. doi: 10.1038/516165a. PMID: 25503219. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
189. Broekhuysen J., Stockis A., Lins R.L., De Graeve J., Rossignol J.F. Nitazoxanide: pharmacokinetics and metabolism in man. Int. J. Clin. Pharm. Ther. 2000;38(8):387–394. doi: 10.5414/cpp38387. PMID: 10984012. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
190. Baldo B.A. Side effects of cytokines approved for therapy. Drug Saf. 2014;37(11):921–943. doi: 10.1007/s40264-014-0226-z. PMID: 25270293; PMCID: PMC7101846. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
191. Hsieh C.L., Huang H.S., Chen K.C., Saka T., Chiang C.Y., Chung L.W.K., Sung S.Y. A novel salicylanilide derivative induces autophagy cell death in castration-resistant prostate cancer via ER stress-activated PERK signaling pathway. Mol. Cancer Therapeut. 2020;19(1):101–111. doi: 10.1158/1535-7163.MCT-19-0387. PMID: 31530650. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
192. Hu M., Ye W., Li J., Zhou P., Chu Z., Huang W. The salicylanilide derivatives inhibit signal transducer and activator of transcription 3 pathways in A549 lung cancer cells. Anti Cancer Drugs. 2016;27(1):41–47. doi: 10.1097/CAD.0000000000000303. PMID: 26469835. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
193. Al Zaid Siddiquee K., Turkson J. STAT3 as a target for inducing apoptosis in solid and hematological tumors. Cell Res. 2008;18(2):254–267. doi: 10.1038/cr.2008.18. PMID: 18227858; PMCID: PMC2610254. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
194. Qin J.J., Yan L., Zhang J., Zhang W.D. STAT3 as a potential therapeutic target in triple negative breast cancer: a systematic review. J. Exp. Clin. Cancer Res. 2019;38(1):195. doi: 10.1186/s13046-019-1206-z. PMID: 31088482; PMCID: PMC6518732. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
195. Gargantilla M., Persoons L., Kauerová T., del Río N., Daelemans D., Priego E.-M., Kollar P., Pérez-Pérez M.-J. Hybridization approach to identify salicylanilides as inhibitors of tubulin polymerization and signal transducers and activators of transcription 3 (STAT3) Pharmaceuticals. 2022;15(7):835. doi: 10.3390/ph15070835. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
196. Marrugal-Lorenzo J.A., Serna-Gallego A., Berastegui-Cabrera J., Pachón J., Sánchez-Céspedes J. Repositioning salicylanilide anthelmintic drugs to treat adenovirus infections. Sci. Rep. 2019;9(1):17. doi: 10.1038/s41598-018-37290-3. PMID: 30626902; PMCID: PMC6327057. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
197. Rossignol J.F., Bardin M.C., Fulgencio J., Mogelnicki D., Bréchot C. A randomized double-blind placebo-controlled clinical trial of nitazoxanide for treatment of mild or moderate COVID-19. EClinicalMedicine. 2022;45 doi: 10.1016/j.eclinm.2022.101310. PMID: 35237748; PMCID: PMC8883002. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
198. Jeon S., Ko M., Lee J., Choi I., Byun S.Y., Park S., Shum D., Kim S. Identification of antiviral drug candidates against SARS-CoV-2 from FDA-approved drugs. Antimicrob. Agents Chemother. 2020;64(7):e00819–e00820. doi: 10.1128/AAC.00819-20. PMID: 32366720; PMCID: PMC7318052. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
199. Al-Kuraishy H.M., Al-Gareeb A.I., Alzahrani K.J., Alexiou A., Batiha G.E. Niclosamide for Covid-19: bridging the gap. Mol. Biol. Rep. 2021;48(12):8195–8202. doi: 10.1007/s11033-021-06770-7. PMID: 34664162; PMCID: PMC8522539. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
200. Firth A., Prathapan P. Broad-spectrum therapeutics: a new antimicrobial class. Curr Res Pharmacol Drug Discov. 2021;2 doi: 10.1016/j.crphar.2020.100011. PMID: 34870144; PMCID: PMC8035643. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
201. Aimo A., Baritussio A., Emdin M., Tascini C. Amiodarone as a possible therapy for coronavirus infection. Eur J Prev Cardiol. 2021;28(12):e16–e18. doi: 10.1177/2047487320919233. PMID: 32295404; PMCID: PMC7928952. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
202. Blaess M., Kaiser L., Sauer M., Csuk R., Deigner H.P. COVID-19/SARS-CoV-2 infection: lysosomes and lysosomotropism implicate new treatment strategies and personal risks. Int. J. Mol. Sci. 2020;21(14):4953. doi: 10.3390/ijms21144953. PMID: 32668803; PMCID: PMC7404102. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
203. Breiden B., Sandhoff K. Emerging mechanisms of drug-induced phospholipidosis. Biol. Chem. 2019;401(1):31–46. doi: 10.1515/hsz-2019-0270. Erratum in: Biol Chem. 2021;403(2):251. PMID: 31408430. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
204. Koh H.X., Aye H.M., Tan K.S., He C.Y. The lysosomotropic drug LeuLeu-OMe induces lysosome disruption and autophagy-independent cell death in Trypanosoma brucei. Microb Cell. 2015;2(8):288–298. doi: 10.15698/mic2015.08.217. PMID: 28357304; PMCID: PMC5349101. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
205. Rabinovitch M., Zilberfarb V., Ramazeilles C. Destruction of Leishmania mexicana amazonensis amastigotes within macrophages by lysosomotropic amino acid esters. J. Exp. Med. 1986;163(3):520–535. doi: 10.1084/jem.163.3.520. PMID: 3950542; PMCID: PMC2188052. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
206. Ch’ng J.H., Liew K., Goh A.S., Sidhartha E., Tan K.S. Drug-induced permeabilization of parasite’s digestive vacuole is a key trigger of programmed cell death in Plasmodium falciparum. Cell Death Dis. 2011;2(10):e216. doi: 10.1038/cddis.2011.97. PMID: 21993392; PMCID: PMC3219093. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
207. Salata C., Calistri A., Parolin C., Baritussio A., Palù G. Antiviral activity of cationic amphiphilic drugs. Expert Rev. Anti Infect. Ther. 2017;15(5):483–492. doi: 10.1080/14787210.2017.1305888. PMID: 28286997; PMCID: PMC7103695. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
208. Norinder U., Tuck A., Norgren K., Munic Kos V. Existing highly accumulating lysosomotropic drugs with potential for repurposing to target COVID-19. Biomed. Pharmacother. 2020;130 doi: 10.1016/j.biopha.2020.110582. PMID: 32763818; PMCID: PMC7392152. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
209. Ekins S., Lane T.R., Madrid P.B. Tilorone: a broad-spectrum antiviral invented in the USA and commercialized in Russia and beyond. Pharm. Res. (N. Y.) 2020;37(4):71. doi: 10.1007/s11095-020-02799-8. Erratum in: Pharm Res. 2020 Nov 6;37(12):239. PMID: 32215760; PMCID: PMC7100484. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
210. Puhl A.C., Fritch E.J., Lane T.R., Tse L.V., Yount B.L., Sacramento C.Q., Tavella T.A., Costa F.T.M., Weston S., Logue J., Frieman M., Premkumar L., Pearce K.H., Hurst B.L., Andrade C.H., Levi J.A., Johnson N.J., Kisthardt S.C., Scholle F., Souza T.M.L., Moorman N.J., Baric R.S., Madrid P., Ekins S. 2020 Dec 2:2020. Repurposing the Ebola and Marburg Virus Inhibitors Tilorone, Quinacrine and Pyronaridine: in Vitro Activity against SARS-CoV-2 and Potential Mechanisms. bioRxiv [Preprint] 12.01.407361. doi: 10.1101/2020.12.01.407361. Update in: ACS Omega. 2021 Mar 10;6(11):7454-7468. PMID: 33299990; PMCID: PMC7724658. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [Google Scholar (opens in a new tab)]
211. Boriskin Y.S., Leneva I.A., Pécheur E.I., Polyak S.J. Arbidol: a broad-spectrum antiviral compound that blocks viral fusion. Curr. Med. Chem. 2008;15(10):997–1005. doi: 10.2174/092986708784049658. PMID: 18393857. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
212. Alavi Darazam I., Shokouhi S., Mardani M., Pourhoseingholi M.A., Rabiei M.M., Hatami F., Shabani M., Moradi O., Gharehbagh F.J., Irvani S.S.N., Amirdosara M., Hajiesmaeili M., Rezaei O., Khoshkar A., Lotfollahi L., Gachkar L., Dehbsneh H.S., Khalili N., Soleymaninia A., Kusha A.H., Shoushtari M.T., Torabinavid P. Umifenovir in hospitalized moderate to severe COVID-19 patients: a randomized clinical trial. Int. Immunopharm. 2021;99 doi: 10.1016/j.intimp.2021.107969. PMID: 34273635; PMCID: PMC8270750. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
213. Nojomi M., Yassin Z., Keyvani H., Makiani M.J., Roham M., Laali A., Dehghan N., Navaei M., Ranjbar M. Effect of Arbidol (Umifenovir) on COVID-19: a randomized controlled trial. BMC Infect. Dis. 2020;20(1):954. doi: 10.1186/s12879-020-05698-w. PMID: 33317461; PMCID: PMC7734453. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
214. Munić V., Banjanac M., Koštrun S., Nujić K., Bosnar M., Marjanović N., Ralić J., Matijašić M., Hlevnjak M., Eraković Haber V. Intensity of macrolide anti-inflammatory activity in J774A.1 cells positively correlates with cellular accumulation and phospholipidosis. Pharmacol. Res. 2011;64(3):298–307. doi: 10.1016/j.phrs.2011.03.011. PMID: 21473915. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
215. Tummino T.A., Rezelj V.V., Fischer B., Fischer A., O’Meara M.J., Monel B., Vallet T., Zhang Z., Alon A., O’Donnell H.R., Lyu J., Schadt H., White K.M., Krogan N.J., Urban L., Shokat K.M., Kruse A.C., García-Sastre A., Schwartz O., Moretti F., Vignuzzi M., Pognan F., Shoichet B.K. 2021. Phospholipidosis Is a Shared Mechanism Underlying the in Vitro Antiviral Activity of Many Repurposed Drugs against SARS-CoV-2. bioRxiv [Preprint] Mar 24:2021.03.23.436648. doi: 10.1101/2021.03.23.436648. PMID: 33791693; PMCID: PMC8010720. [Google Scholar (opens in a new tab)]
216. Lane T.R., Ekins S. Defending antiviral cationic amphiphilic drugs that may cause drug-induced phospholipidosis. J. Chem. Inf. Model. 2021;61(9):4125–4130. doi: 10.1021/acs.jcim.1c00903. PMID: 34516123; PMCID: PMC8576745. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
217. Shameer K., Glicksberg B.S., Hodos R., Johnson K.W., Badgeley M.A., Readhead B., Tomlinson M.S., O’Connor T., Miotto R., Kidd B.A., Chen R., Ma’ayan A., Dudley J.T. Systematic analyses of drugs and disease indications in RepurposeDB reveal pharmacological, biological and epidemiological factors influencing drug repositioning. Briefings Bioinf. 2018;19(4):656–678. doi: 10.1093/bib/bbw136. PMID: 28200013; PMCID: PMC6192146. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
218. Varalda M., Antona A., Bettio V., Roy K., Vachamaram A., Yellenki V., Massarotti A., Baldanzi G., Capello D. Psychotropic drugs show anticancer activity by disrupting mitochondrial and lysosomal function. Front. Oncol. 2020;10 doi: 10.3389/fonc.2020.562196. PMID: 33194631; PMCID: PMC7604408. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
219. Lamb R., Ozsvari B., Lisanti C.L., Tanowitz H.B., Howell A., Martinez-Outschoorn U.E., Sotgia F., Lisanti M.P. Antibiotics that target mitochondria effectively eradicate cancer stem cells, across multiple tumor types: treating cancer like an infectious disease. Oncotarget. 2015;6(7):4569–4584. doi: 10.18632/oncotarget.3174. PMID: 25625193; PMCID: PMC4467100. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
220. Napolitano F., Zhao Y., Moreira V.M., Tagliaferri R., Kere J., D’Amato M., Greco D. Drug repositioning: a machine-learning approach through data integration. J. Cheminf. 2013;5(1):30. doi: 10.1186/1758-2946-5-30. PMID: 23800010; PMCID: PMC3704944. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
221. Sugawara A., Shima H., Sueki A., Hirose T., Matsui H., Nakano H., Hanaki H., Akagawa K.S., Ōmura S., Sunazuka T. Non-antibiotic 12-membered macrolides: design, synthesis and biological evaluation in a cigarette-smoking model. J. Antibiot. (Tokyo) 2016;69(4):319–326. doi: 10.1038/ja.2015.91. PMID: 26419414. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
222. Hodge S., Tran H.B., Hamon R., Roscioli E., Hodge G., Jersmann H., Ween M., Reynolds P.N., Yeung A., Treiberg J., Wilbert S. Nonantibiotic macrolides restore airway macrophage phagocytic function with potential anti-inflammatory effects in chronic lung diseases. Am. J. Physiol. Lung Cell Mol. Physiol. 2017;312(5):L678–L687. doi: 10.1152/ajplung.00518.2016. PMID: 28258107; PMCID: PMC5451592. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
223. Lusamba Kalonji N., Nomura K., Kawase T., Ota C., Kubo H., Sato T., Yanagisawa T., Sunazuka T., Ōmura S., Yamaya M. The non-antibiotic macrolide EM900 inhibits rhinovirus infection and cytokine production in human airway epithelial cells. Phys. Rep. 2015;3(10) doi: 10.14814/phy2.12557. PMID: 26462747; PMCID: PMC4632947. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
224. Liu K.C., Fang J.M., Jan J.T., Cheng T.J., Wang S.Y., Yang S.T., Cheng Y.S., Wong C.H. Enhanced anti-influenza agents conjugated with anti-inflammatory activity. J. Med. Chem. 2012;55(19):8493–8501. doi: 10.1021/jm3009844. PMID: 22963087. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
225. Shaker A.M.M., Abdelall E.K.A., Abdellatif K.R.A., Abdel-Rahman H.M. Synthesis and biological evaluation of 2-(4-methylsulfonyl phenyl) indole derivatives: multi-target compounds with dual antimicrobial and anti-inflammatory activities. BMC Chem. 2020;14(1):23. doi: 10.1186/s13065-020-00675-5. PMID: 32259135; PMCID: PMC7106896. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
226. Derendorf H. Excessive lysosomal ion-trapping of hydroxychloroquine and azithromycin. Int. J. Antimicrob. Agents. 2020;55(6) doi: 10.1016/j.ijantimicag.2020.106007. PMID: 32389720; PMCID: PMC7204663. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
227. Pirofski L.A., Casadevall A. The damage-response framework of microbial pathogenesis and infectious diseases. Adv. Exp. Med. Biol. 2008;635:135–146. doi: 10.1007/978-0-387-09550-9_11. PMID: 18841709; PMCID: PMC7123708. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
228. Blakley B.R., Rousseaux C.G. Effect of ivermectin on the immune response in mice. Am. J. Vet. Res. 1991;52(4):593–595. PMID: 1828942. [PubMed (opens in a new tab)] [Google Scholar (opens in a new tab)]
229. Daminelli S., Haupt V.J., Reimann M., Schroeder M. Drug repositioning through incomplete bi-cliques in an integrated drug-target-disease network. Integr Biol (Camb). 2012;4(7):778–788. doi: 10.1039/c2ib00154c. PMID: 22538435. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
230. Watanabe S.M., Ehrlich L.S., Strickland M., Li X., Soloveva V., Goff A.J., Stauft C.B., Bhaduri-McIntosh S., Tjandra N., Carter C. Selective targeting of virus replication by proton pump inhibitors. Sci. Rep. 2020;10(1):4003. doi: 10.1038/s41598-020-60544-y. PMID: 32132561; PMCID: PMC7055211. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
231. Hopkins A.L. Network pharmacology: the next paradigm in drug discovery. Nat. Chem. Biol. 2008;4(11):682–690. doi: 10.1038/nchembio.118. PMID: 18936753. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
232. Parisi D., Adasme M.F., Sveshnikova A., Bolz S.N., Moreau Y., Schroeder M. Drug repositioning or target repositioning: a structural perspective of drug-target-indication relationship for available repurposed drugs. Comput. Struct. Biotechnol. J. 2020;18:1043–1055. doi: 10.1016/j.csbj.2020.04.004. PMID: 32419905; PMCID: PMC7215100. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
233. Adasme M.F., Parisi D., Sveshnikova A., Schroeder M. Structure-based drug repositioning: potential and limits. Semin. Cancer Biol. 2021;68:192–198. doi: 10.1016/j.semcancer.2020.01.010. PMID: 32032699. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
234. Sauer A., Peukert K., Putensen C., Bode C. Antibiotics as immunomodulators: a potential pharmacologic approach for ARDS treatment. Eur. Respir. Rev. 2021;30(162) doi: 10.1183/16000617.0093-2021. PMID: 34615700. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
235. Chitalia V.C., Munawar A.H. A painful lesson from the COVID-19 pandemic: the need for broad-spectrum, host-directed antivirals. J. Transl. Med. 2020;18(1):390. doi: 10.1186/s12967-020-02476-9. PMID: 33059719; PMCID: PMC7558548. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
236. Webb B.A., Chimenti M., Jacobson M.P., Barber D.L. Dysregulated pH: a perfect storm for cancer progression. Nat. Rev. Cancer. 2011;11(9):671–677. doi: 10.1038/nrc3110. PMID: 21833026. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
237. Takenaka T. Classical vs reverse pharmacology in drug discovery. BJU Int. 2001;88(Suppl 2):7–10. doi: 10.1111/j.1464-410x.2001.00112.x. discussion 49-50, PMID: 11589663. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
238. Ringel M.S., Scannell J.W., Baedeker M., Schulze U. Breaking eroom’s law. Nat. Rev. Drug Discov. 2020;19(12):833–834. doi: 10.1038/d41573-020-00059-3. PMID: 32300238. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
239. Campbell W.C. In: In Inventive Minds. Weber R.J., Perkins D.N., editors. Oxford University Press; New York: 1992. The genesis of the antiparasitic drug ivermectin; pp. 194–214. [Google Scholar (opens in a new tab)]
240. Tyteca D., Van Der Smissen P., Van Bambeke F., Leys K., Tulkens P.M., Courtoy P.J., Mingeot-Leclercq M.P. Azithromycin, a lysosomotropic antibiotic, impairs fluid-phase pinocytosis in cultured fibroblasts. Eur. J. Cell Biol. 2001;80(7):466–478. doi: 10.1078/0171-9335-00180. PMID: 11499789. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
241. Kuo H.H., Kakadiya R., Wu Y.C., Su T.L., Lee T.C., Lin Y.W., Yih L.H. Derivatives of 6-cinnamamido-quinoline-4-carboxamide impair lysosome function and induce apoptosis. Oncotarget. 2016;7(25):38078–38090. doi: 10.18632/oncotarget.9348. PMID: 27191263; PMCID: PMC5122373. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
242. Humeau J., Leduc M., Cerrato G., Loos F., Kepp O., Kroemer G. Phosphorylation of eukaryotic initiation factor-2α (eIF2α) in autophagy. Cell Death Dis. 2020;11(6):433. doi: 10.1038/s41419-020-2642-6. PMID: 32513922; PMCID: PMC7280501. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
243. Tian A.L., Wu Q., Liu P., Zhao L., Martins I., Kepp O., Leduc M., Kroemer G. Lysosomotropic agents including azithromycin, chloroquine and hydroxychloroquine activate the integrated stress response. Cell Death Dis. 2021;12(1):6. doi: 10.1038/s41419-020-03324-w. PMID: 33414432; PMCID: PMC7790317. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
244. Giacometti A., Cirioni O., Barchiesi F., Ancarani F., Scalise G. Activity of nitazoxanide alone and in combination with azithromycin and rifabutin against Cryptosporidium parvum in cell culture. J. Antimicrob. Chemother. 2000;45(4):453–456. doi: 10.1093/jac/45.4.453. PMID: 10747821. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
245. Tamomh A.G., Agena A.M., Elamin E., Suliman M.A., Elmadani M., Omara A.B., Musa S.A. Prevalence of cryptosporidiosis among children with diarrhoea under five years admitted to Kosti teaching hospital, Kosti City, Sudan. BMC Infect. Dis. 2021;21(1):349. doi: 10.1186/s12879-021-06047-1. PMID: 33853528; PMCID: PMC8048339. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
246. Lee S., Beamer G., Tzipori S. The piglet acute diarrhea model for evaluating efficacy of treatment and control of cryptosporidiosis. Hum. Vaccines Immunother. 2019;15(6):1445–1452. doi: 10.1080/21645515.2018.1498436. PMID: 30036127; PMCID: PMC6663130. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
247. Kelleni M.T. Nitazoxanide/azithromycin combination for COVID-19: a suggested new protocol for early management. Pharmacol. Res. 2020;157 doi: 10.1016/j.phrs.2020.104874. PMID: 32360581; PMCID: PMC7192107. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
248. Kelleni M.T. NSAIDs and Kelleni’s protocol as potential early COVID-19 treatment game changer: could it be the final countdown? Inflammopharmacology. 2022;30(1):343–348. doi: 10.1007/s10787-021-00896-7. PMID: 34822026; PMCID: PMC8613510. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
249. de Lemos Neto M., Alexandre R.C.V., Morra R.O.G., da Paz J.A.S., Barroso S.P.C., Resende A.C., de Medeiros-Lima D.J.M., Alexandre P.C.B. Use of glucocorticoids and azithromycin in the therapy of COVID-19. Pharmacol. Rep. 2021;73(6):1513–1519. doi: 10.1007/s43440-021-00286-4. PMID: 34085181; PMCID: PMC8175191. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
250. 2022 May 26. https://www.pharmaceutical-technology.com/news/hyundai-monkeypox-drug-fda/ (opens in a new tab) Online.
251. Peng C., Zhou Y., Cao S., Pant A., Campos Guerrero M.L., McDonald P., Roy A., Yang Z. Identification of vaccinia virus inhibitors and cellular functions necessary for efficient viral replication by screening bioactives and FDA-approved drugs. Vaccines. 2020;8(3):401. doi: 10.3390/vaccines8030401. PMID: 32708182; PMCID: PMC7564539. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
252. 2021 Dec 8. https://www.pharmaceutical-technology.com/news/hyundai-combination-therapy-covid/ (opens in a new tab) Online.
253. Hickson S.E., Margineantu D., Hockenbery D.M., Simon J.A., Geballe A.P. Inhibition of vaccinia virus replication by nitazoxanide. Virology. 2018;518:398–405. doi: 10.1016/j.virol.2018.03.023. PMID: 29625403; PMCID: PMC5929478. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
254. de Gans J., van de Beek D. European dexamethasone in adulthood bacterial meningitis study investigators. Dexamethasone in adults with bacterial meningitis. N. Engl. J. Med. 2002;347(20):1549–1556. doi: 10.1056/NEJMoa021334. PMID: 12432041. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
255. van de Beek D., Brouwer M.C., Koedel U., Wall E.C. Steroid use in non-pneumococcal and non-Haemophilus bacterial meningitis - authors’ reply. Lancet. 2022;399(10326):718. doi: 10.1016/S0140-6736(21)02662-3. PMID: 35183295. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
256. Johns M., George S., Taburyanskaya M., Poon Y.K. A review of the evidence for corticosteroids in COVID-19. J. Pharm. Pract. 2022;35(4):626–637. doi: 10.1177/0897190021998502. PMID: 33719698. [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
257. Inaba H., Pui C.H. Glucocorticoid use in acute lymphoblastic leukaemia. Lancet Oncol. 2010;11(11):1096–1106. doi: 10.1016/S1470-2045(10)70114-5. PMID: 20947430; PMCID: PMC3309707. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
258. Blum V.F., Cimerman S., Hunter J.R., Tierno P., Lacerda A., Soeiro A., Cardoso F., Bellei N.C., Maricato J., Mantovani N., Vassao M., Dias D., Galinskas J., Janini L.M.R., Santos-Oliveira J.R., Da-Cruz A.M., Diaz R.S. Nitazoxanide superiority to placebo to treat moderate COVID-19 - a Pilot prove of concept randomized double-blind clinical trial. EClinicalMedicine. 2021;37 doi: 10.1016/j.eclinm.2021.100981. Erratum in: EClinicalMedicine. 2021 Nov;41:101203. PMID: 34222847; PMCID: PMC8235996. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
259. Singh S., Weiss A., Goodman J., Fisk M., Kulkarni S., Lu I., Gray J., Smith R., Sommer M., Cheriyan J. Niclosamide-A promising treatment for COVID-19. Br. J. Pharmacol. 2022;179(13):3250–3267. doi: 10.1111/bph.15843. PMID: 35348204; PMCID: PMC9111792. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
260. Rai M., Kon K., Ingle A., Duran N., Galdiero S., Galdiero M. Broad-spectrum bioactivities of silver nanoparticles: the emerging trends and future prospects. Appl. Microbiol. Biotechnol. 2014;98(5):1951–1961. doi: 10.1007/s00253-013-5473-x. PMID: 24407450; PMCID: PMC7080016. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
261. Prathapan P. A determination of pan-pathogen antimicrobials? Med. Drug Discov. 2022;14 doi: 10.1016/j.medidd.2022.100120. PMID: 35098103; PMCID: PMC8785259. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]
262. Alegría-Arcos M., Barbosa T., Sepúlveda F., Combariza G., González J., Gil C., Martínez A., Ramírez D. Network pharmacology reveals multitarget mechanism of action of drugs to be repurposed for COVID-19. Front Pharmacol. 2022;13:952192. doi: 10.3389/fphar.2022.952192. PMID: 36052135; PMCID: PMC9424758. [PMC free article (opens in a new tab)] [PubMed (opens in a new tab)] [CrossRef (opens in a new tab)] [Google Scholar (opens in a new tab)]